I. INTRODUCTION
Despite certain successes in studying the processes of evolution of living and non-living nature from the standpoint of nonequilibrium thermodynamics [1-9], bioenergetics [10-15] and synergetics [16-20], an obvious contradiction of not only classical, but also nonequilibrium thermodynamics the nature of biological evolution "is preserved. Interpretation of the second principle as a principle of increasing entropy imposes "thermal death" on the Universe, and degradation on any of its closed parts [21]. Attempts to consider evolution as a random process [22], the result of the emergence of "order" from "chaos" [19] and even more so "consumption of negentropy" [11] did not give satisfactory results. The very concept of "self-organization" of systems, understood as a spontaneous (not imposed from the outside) ordering of the system [21], is in "blatant" contradiction with the principle of "self-infringement of equilibrium" of classical thermodynamics. Attempts to "explain" the emergence of anti-dissipative thermomechanical, thermochemical, thermoelectric, thermomagnetic, thermo-galvanomagnetic, etc. effects as manifestations of "synergetism" - the superposition of dissipative processes [2, 3].
A way out can be found from the standpoint of a more general theory of transfer and transformation processes of any forms of energy [23], developed and supplemented later in the monographs "Thermokinetics" [24] and "Energodynamics" [25]. Unlike W. Thomson's "pseudothermodynamics" [25] or L. Onsager's "quasithermodynamics" [26], this theory does not exclude from consideration any (irreversible or reversible) part of the phenomenon under study and covers the entire range of real processes - from quasireversible to extremely irreversible. This is achieved by finding the driving forces of these processes Xi and their speeds (flows Ji), directly on the basis of the law of conservation of energy, generalized to systems that are far from equilibrium. This opens up new possibilities for the application of thermodynamics to the study of biosystems and eliminates its contradictions with the laws of biological evolution.
II. METHODOLOGICAL FEATURES OF ENERGODYNAMICS
The fundamental difference between enerodynamics and thermodynamics of the irreversible processes (TIP) and other fundamental disciplines is its ability to consider nonequilibrium systems as a whole, without dividing them into an infinite number of elementary volumes , assumed to be homogeneous. This allows you to preserve the so-called system-forming connections inherent in the biosystem as a whole but absent in its individual parts. It is these properties that distinguish a living organism from a simple set of organs (subsystems) or mass elements that are formed during such fragmentation. In view of the inevitable disruption of the functions of individual organs when the organism is divided into volume elements, attempts to restore the system-forming properties lost at the same time by finding "suitable integrals" are doomed to failure. The realization of this circumstance was, according to A. Poincaré, "the greatest shock that physics experienced since the time of I. Newton" [28].
Another methodological feature of energy dynamics is taking into account the opposite direction of processes in different parts (areas, phases, components) of a nonequilibrium system, which makes such processes irreversible even when they are quasi-static (infinitely slow). This can be verified by selecting subsystems with volumes and in a non-uniform object of study, within which the density of any extensive parameter of the system (its mass , number of moles -th substances or phases , entropy , charge , components of momentum and its moment , etc.) is greater or less than their average value . Then, by virtue of the obvious equality we have:
Hence it follows that in a non-uniform system there are always subsystems (areas, phases, components) in which this deviation of and has the opposite sign. The law of "unity and struggle of opposites."
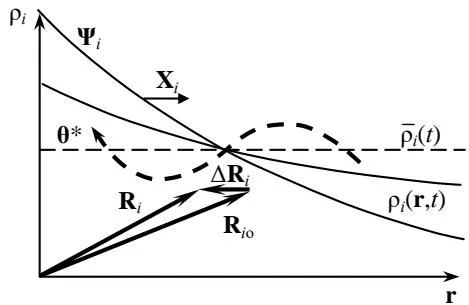
Another methodological feature of energy dynamics is the refusal to use in the foundations of the theory of hypotheses, postulates, model representations and considerations of the molecular-kinetic and statistical-mechanical theory, including the hypothesis of local equilibrium by I. Prigogine, which lies at the basis of the TIP. According to this hypothesis, the volume elements of a non-equilibrium system as a whole are in local equilibrium (despite the occurrence of dissipative processes in them), so that their state can be described by the same number of variables as in equilibrium (despite the appearance of local "thermodynamic forces" ), and all equations of classical thermodynamics are applicable to them (despite their inevitable transition into inequalities). Contrary to this hypothesis, additional parameters of nonequilibrium of the systems under study are introduced in energy dynamics. The necessity of their introduction is proved by the "principle of definiteness", according to which the number of independent arguments of the internal energyas a function of the state of the system is equal to the number of independent processes occurring in it. This principle, which is proved in energy dynamics "by contradiction," requires the introduction of additional coordinates of vector relaxation processes that cause a "redistribution" of extensive parametersover the volume of the system. To find these coordinates, consider an arbitrary system with an inhomogeneous densityof any extensive parameter, considered as a quantitative measure of the i-th energy carrier(Fig. 1). As follows from the figure, whendeviates from the average value, a certain amountof the energy carrieris transferred from one part of the system to another in the direction indicated by the dotted arrow. Such "redistribution" of the extensive valuecauses a shift in the center of its value from the initial positionto the current one. In this case, a certain "moment of distribution"arises:
with a shoulder , called in energy dynamics "displacement vector" [25].
Since in a homogeneous state, the state of the nonequilibrium system as a whole is characterized in the first approximation by a doubled number of state variables and , i.e., . In this case, its total differential can be represented as an identity [25]:
where is the average value of the generalized potential (absolute temperature and pressure , chemical , electric , gravitational and other potentials); is the forces in their general physical understanding as a gradient of the -th form of energy with the opposite sign, the specific value of which corresponds to the concept of thermodynamic force in its "energy" representation [29].
The members of the 1st sum in expression (3) are in conditions of constancy of , that is, in the absence of redistribution processes. This means that the local potentials in such processes change to the same extent in all parts of the system (as well as in homogeneous systems). This kind of change in state is reminiscent of a uniform fall of precipitation on an uneven surface. Their particular case is the equilibrium (reversible) processes of heat and mass transfer of the system, the work of introducing -th substances or charge into the system, its all-round compression or expansion, etc. do not determine the heat or work of the process, as was the case in the case of reversible processes. On the contrary, from the very beginning it is recognized that the variables are emergent quantities, that is, they can change in the general case both due to external energy exchange and due to internal sources during the course of internal spontaneous processes. This is reflected in the equations of the balance of these quantities, which are similar in meaning to the equations of the balance of entropy. This approach means refusal to calculate the external energy exchange of the system by changing the parameters , and the transition to direct measurement of energy carrier fluxes through the boundaries of the system , where .
The second sum of identity (3), on the contrary, owes its origin to the spatial heterogeneity of the systems under study. Its terms also characterize the elementary work of the same kind as in mechanics, which is determined by the product of the resulting force of the -th kind by the displacement caused by it of the object of its application (in this case, the value ). This work is different from those included in the first sum (3). Since the forces in (3) are under the conditions of constant parameters , then , where . The work performed by the forces or consists in the redistribution of the energy carrier over the volume of the system. Thus, energy dynamics introduces into consideration a new class of transfer processes that have a vector (directed, ordered) character.
In the particular case of homogeneous systems , expression (3) turns into the combined equation of the 1st and 2nd principles of classical thermodynamics of open systems in the form of the Gibbs relation [21]:
where is the number of independent energy carriers of the system.
At the same time, a unique feature of energy dynamics consists in obtaining many non-trivial consequences even before its application to specific systems. The latter, as is known, requires the use of uniqueness conditions, in that knowledge of the thermophysical properties of the object, its equations of state and transfer, boundary conditions, etc. Therefore, the consequences obtained directly from identity (4), before using the uniqueness conditions, acquire the status immutable truths.
III. FINDING DRIVING FORCES AND GENERALIZED SPEEDS OF BIOLOGICAL PROCESSES IN ENERGODYNAMICS
In contrast to the existing linear TIP, energy dynamics introduces thermodynamic forces and flows of energy carrier on a more general basis of the law of conservation of energy, and not the principle of increasing entropy. In L. Onsager's "quasithermodynamics" [27] dealing with relaxation processes, their scalar analogs and are found from the expression for the rate of entropy increase in an adiabatically isolated system :
where is "thermodynamic force" as a measure of the deviation of some -th parameter of the system from its equilibrium value ; is the generalized rate of the -th relaxation process.
However, since the parameters are obviously absent in equilibrium thermodynamics, Onsager's theory was a kind of formalism that has nothing to do with reality. The situation changed when I. Prigogine proposed to move on to the study of the so-called "stationary irreversible processes", in which the parameters and acquire a vector nature and are maintained unchanged by means of "external compulsion", that is, performing work on the system against equilibrium". In this case, the parameters and can be found from disciplines operating with the concept of work, by separating from that part of it that is responsible for the "production of entropy" and is numerically equal to the work done on the system . However, this required the compilation of cumbersome equations for the balance of energy, mass, charge, momentum, entropy, etc. in order to isolate from them the irreversible part of the process associated with the production of entropy . This most time-consuming part of the TIP application required from the user not only an outstanding knowledge of the relevant fundamental disciplines, but also the application of a number of hypotheses, since these disciplines were deliberately limited to the consideration of conservative (nondissipative) systems and did not contain dissipative terms. This was the main reason why teaching consumer goods in higher education turned out to be unrealistic.
The situation is completely different in energy dynamics, where the sought forces and fluxes are already contained in its basic identity (3). At the same time, the arbitrariness inherent in TIP in the choice of driving forces and generalized speeds of transfer processes is eliminated, and the concept of force and generalized speed of the process becomes the same for all disciplines. So, if the first sum (3) includes the term , which characterizes reversible heat transfer in the combined equation of the 1st and 2nd principles of classical thermodynamics, then the term , will appear in the 2nd sum (3), where is the specific "thermotive" force, is the entropy flux. Similarly, if the first sum (3) includes the term , which characterizes the reversible work of expansion, then in the second sum (3) there will appear an additional term , which characterizes the process of contraction of some and expansion of other parts systems, for example, the ventricle and atrium ( is volumetric flow). In the same way, if the first sum (3) includes the term , which characterizes the reversible transfer of the -th substance through the boundaries of the system, then in the second sum (3) there will appear a term , which characterizes the work separation of this substance in the cell membrane or in the dialyzer ( is the flow of the th substance). Similarly, driving forces can be found in so-called "complex" systems that perform other types of work besides expansion work. So, if the term is included in the 1st sum (3), which characterizes the reversible work of introducing an electric charge into the region with an average electric potential , then in the second sum (3) the term , creating the elementary work of separating charges in the cell membrane or in a galvanic cell ( is electric field strength, - electric current).
It is easy to see that the terms of the second sum (3) can have different signs depending on whether the system is doing work or work is being done on the system. This is the fundamental difference between the proposed method and TIP, in which the terms are always positive (as well as "entropy production"). Meanwhile, in biosystems that consume free energy from the environment, , which contradicts (5) and leads to absurdities such as "negentropy production". In addition to eliminating it, this approach allows energy dynamics to study real processes, not excluding from consideration any (reversible or irreversible) component.
A significant advantage of this approach is also that it eliminates the need to draw up cumbersome equations for the balance of energy, mass, charge, momentum, entropy, etc. It is also important that energy dynamics acquires the ability to reflect on a quantitative and qualitative level the emergence of new (emergent) properties in the system. Indeed, the parameters are absent in equilibrium systems and their elements, and arise only when they deviate from a uniform state. Thus, energy dynamics is distinguished by taking into account not only the local nonequilibrium of the studied systems , but also the ability to reflect the evolution of biosystems, which consists in the appearance of new properties in them. In the future, this also makes it possible to substantiate the dialectical unity of the processes of evolution and involution [30]. In addition, the unity of the dimensions of forces of various natures opens up the possibility of finding their resultant , which subsequently makes it possible to significantly simplify the transport equations.
IV. CORRECTION OF THE EQUATIONS OF "PASSIVE TRANSPORT" IN BIOSYSTEMS
In L. Onsager's "quasi-thermodynamics" [27], it is postulated that each of the fluxes linearly depends on all thermodynamic acting in the system forces . The corresponding equations are called the "phenomenological laws of Onsager":
Here is constant (independent of ) kinetic coefficients, called phenomenological and obeying the so-called "reciprocity relations" Onsager . These ratios reflect, in his opinion, the interconnection of the flows, which is the reason for the appearance of the aforementioned "side" effects of their "overlap".
According to (6), the terms of the flow have the same sign. This is natural for the case of purely dissipative processes, when the total rate of approach of the system to equilibrium is the sum of the rates of individual relaxation processes. Meanwhile, a class of so-called "conjugate" processes is known, when some of them proceed in the direction of equilibrium, while others, on the contrary, remove it from equilibrium. Such, for example, are the Belousov-Zhabotinsky cyclic reactions called "chemical clocks" [31], "active transport" in biosystems (transfer of substances to the region of increased reaction affinity) [32], "ascending diffusion" in metals and alloys [33], the processes of concentration of matter in the Universe [30], etc. This means that at least some of the forces and flows have the opposite sign, that is, when some i-th relaxation process occurs, the system moves away from equilibrium on other, j-th degrees of freedom. In other words, along with dissipative phenomena in such systems, processes of opposite direction are observed. These include, in particular, the transfer of a substance to an area with its increased concentration (the so-called "ascending diffusion"), the phenomenon of "self-organization" of biosystems, processes of structure formation in solutions and melts. The state of equilibrium is possible only by performing useful work on it, we have to admit that in biosystems, along with external work, internal work is performed against some of the forces , which is not associated with the production of entropy. Equations (6) do not take into account this specificity of systems performing useful work. This makes TIP inapplicable to biosystems.
The interpretation of the effects of superposition of heterogeneous processes in consumer goods is also erroneous. Indeed, if the flows in the consumer goods are found as time derivatives of the independent parameters , then they are also independent of each other and therefore cannot interact (overlap). This is especially obvious for stationary states, when part of the "superimposed" flows simply disappears, and the effects of "superimposition" nevertheless take on a maximum value. This means that the explanation of various (thermomechanical, thermoelectric, thermochemical, electromagnetic, etc. effects) in consumer goods as a consequence of the interaction of dissimilar flows, and not the summation of forces, does not correspond to the essence of the matter.
The transfer equations from the standpoint of energy dynamics appear in a completely different light. Like classical thermodynamics, it involves any equations (state or transfer) from the outside as a kind of uniqueness condition describing the properties of specific systems. At the same time, the mathematical apparatus of thermodynamics and energy dynamics, based on the properties of the total differential of a number of state functions, does not depend on these equations. As is known from mechanics, for each independent transfer process there is a unique (resultant) force , which generates this process and disappears when it stops [25]. The components of this force differ in their physical nature, however, unlike , they have the same dimension [N]. If such (resulting) force is found, and laws (6) take the so-called "diagonal" form, similar to the equations of heat conduction, electrical conductivity, diffusion, etc. and does not contain cross terms with [34]:
In this case, Onsager's reciprocity relations are fulfilled trivially ( ) and become redundant, and with them the requirement of linearity of laws (6), which is necessary for their fulfillment. This means that the phenomenological coefficients in (7) can be arbitrary functions of the variables and the forces , while laws (6) in the general case can be nonlinear. In particular, as shown in [24], the laws of passive transport of -th substances take the form:
where are the coefficients of osmotic diffusion of the kth substance, depending on the fields of temperature, pressure and concentration of all independent components of the system; is drop in the chemical potential on the membrane. Meanwhile, in the diffusion laws proposed by Osager himself, the sum appears, as in (5) [27]. In the diagonal form of laws (7.8), their nonlinearity, associated with the variability of the coefficients , no longer interferes with the finding of superposition effects. Let us show this by the example of a biological membrane permeable to the -th substance. Expanding the expression for the total differential of the chemical potential as a function of temperature, pressure and concentrations of all -th independent components of the system ( ), we have:
This means that the transfer equation (6) for discontinuous media in their expanded form has the form:
where , , are temperature, pressure and concentration drops of -th substances on the membrane. The terms of this expression are the components of the resulting force , the first of which is responsible for the phenomenon of thermal diffusion (transfer of matter due to temperature difference), the second - for the phenomenon of barodiffusion (transfer of matter due to pressure difference), and the third - for the phenomenon of ordinary (concentration) diffusion. The mutual compensation of these components of the resulting force is the reason for the onset of a stationary state, which would be more correctly called the state of "partial equilibrium". In this case, the very stationary effects such as are obtained in energy dynamics as a result of the "superposition" of dissimilar forces, not flows.
In particular, from (10) at , regardless of the value of , the well-known expression for the stationary effect of the appearance of the so-called osmotic pressure in a binary isothermal system (the first component is a solvent) follows directly:
Here is the stationary difference in the concentration of the solute on both sides of the biological membrane.
This made it possible to propose a method for studying superposition effects in nonlinear systems [23], which opens up the possibility of studying the kinetics of processes in biosystems that are far from equilibrium.
V. ESTABLISHING THE RELATIONSHIP OF CHEMICAL REACTIONS WITH METABOLIC PROCESSES
When applying the TIP to phenomena of different tensor rank and type, it turned out that, in accordance with the Curie principle (which establishes the conditions for the preservation of bonds during coordinate transformations), the generalized rate of a process in equations of the type (1) can depend only on thermodynamic forces of the same (or even) of tensor rank [1,2]. This meant that the chemical reactions described in TIP by the terms (where is the standard chemical affinity of the rth chemical reaction, is the degree of its completeness), i.e., as scalar processes, cannot interact with the processes of metabolism (exchange substances) having a vector nature. There was an obvious contradiction between TIP and biology, for which it is precisely this interaction that plays a decisive role in the life processes of biosystems. To resolve this contradiction, I. Prigogine put forward the theory of "stationary conjugation", in which the fact of the presence of active transport of substances through biological membranes due to the occurrence of chemical reactions on them was explained by the specificity of stationary states with their inherent ratios between the costs of individual reagents. However, it remained unclear why the aforementioned relationship of chemical reactions with metabolic processes persisted in non-stationary regimes. The answer to this question is given by the basic identity of energy dynamics in the form (4). If the term appears in its first sum, describing the -th scalar chemical reactions in homogeneous media, then in the second sum (4) additional terms of the vector nature , reactors, Van't Hoff boxes, cell reactors, etc.), where ; is the local value of the chemical affinity of the -th chemical reaction in a given cross-section of the flow reactor; is the flow of reagents participating in it. Indeed, for steady-state reactions, the term can be represented as , where is the local value of the driving force of the -th flow chemical reaction; is the coordinate of the "reaction front" in the flow reactor. In this case, the laws of active transport of substances in membranes take the form:
where is the flow of chemically reacting substances through the biological membrane. Thus, under conditions of spatial separation of reagents (as in a Van't Hoff box), chemical reactions acquire a directional (vector) character, which determines their interaction with metabolic processes in full accordance with the Curie principle. In the absence of the transfer of reagents in the field of intermolecular forces, chemical reactions inevitably acquire a dissipative character, which is taken into account in TIP by assigning the term entirely to heat sources. This removes one of the main contradictions between consumer goods and bioenergetics [24].
VI. CRITERIA FOR THE EVOLUTION AND INVOLUTION OF BIOLOGICAL SYSTEMS
In classical and nonequilibrium thermodynamics, there are no parameters or state functions that could be quite general and strict criteria for the development (ontogenesis) and evolution (phylogenesis) of biosystems. Entropy is not applicable for this purpose, since in biosystems exchanging energy and matter with the environment, it can change due to heat transfer or mass transfer and, on the contrary, remain unchanged if the system moves away from equilibrium or approaches it due to the performance of useful work.
As for the well-known thermodynamic potentials such as the Gibbs free energy or Helmholtz , they are defined, strictly speaking, only for closed homogeneous systems and are not applicable in the boundary conditions specified by the flows of matter [27]. It cannot serve as a measure of the ordering of a biosystem and its exergy (technical performance) of extended systems [35], since it depends on the energy supplied from the outside in the process of performing work, as well as on environmental parameters, and is not a function of the state of such systems.
The so-called "production" of entropy (the rate of its increase due to irreversibility) also does not meet these requirements, since this indicator has a minimum only for stationary states of linear systems, and then only near equilibrium [36]. The way out of the situation is again prompted by energetodynamics.
Let us pay attention to the second term (3), which determines the algebraic sum of all types of work (external and internal, useful and dissipative, mechanical and non-mechanical) that can be performed by the open system under study with an arbitrary number of nonequilibrium degrees of freedom . This sum characterizes the transformed (non-equilibrium) part of the internal energy of a spatially heterogeneous system, which we called "energy" (as opposed to the equilibrium, non-workable part of the energy , which we named after Z. Rant (1955) "energy"). Inergy as a non-equilibrium (ordered) part of the internal energy is a function exclusively of the parameters of the spatial inhomogeneity or . According to (3), a homogeneous system cannot perform either external or internal work, since . This means that the measure of the efficiency of the system is precisely the energy as an ordered part of the energy of the system. This allows us to use its change as a very general criterion for the involution of the system, i.e., its degradation as it approaches the state of equilibrium, where :
Here the sign <refers to the relaxation processes of the system; an equal sign - to a state of balance.
On the contrary, the increase in the system's inergy/due to its removal from equilibrium under the influence of external work can serve as a criterion for its evolution:
According to (3), the parameters can be found directly from the known density fields of the corresponding energy carrier , and other parameters of nonequilibrium and are determined from them. All three of these parameters can serve as non-entropy criteria for the evolution of the system [36]. The advantage of these criteria over entropy is that they are able to reflect the evolution of the system for each of its inherent degrees of freedom (mechanical, thermal, baric, chemical, electrical, etc.), and not only its approach to equilibrium, but also distance from it:
This makes it possible to detect the opposite direction of processes not only in different degrees of freedom of the system, but also in its different parts (regions, phases and components) of the system. Since in isolated systems all processes are spontaneous, such an analysis makes meaningful the concept of self-organization of individual degrees of freedom of the system, which does not contradict thermodynamics due to the absence of such for an isolated system as a whole.
VII. DESCRIPTION OF ENERGY CONVERSION PROCESSES IN BIOSYSTEMS
The specificity of energy conversion processes in biosystems is the appearance of additional interrelationships between the rates of dissimilar processes and the flows and of the converted and converted forms of energy. The presence of such a connection is easy to detect on the basis of the law of conservation of energy in the form (3), from which it follows that with a complete transformation of the -th form of energy into the -th
This relationship is reflected by the differential relationships of reciprocity, which are invariably antisymmetric for energy conversion processes [15]:
This (antisymmetric) nature of reciprocity relations is due to the different sign of the work performed by the forces and and does not depend, as shown in [12], on whether these forces belong to even or odd functions of time. In the particular case of linear systems, relations (12) transform into the Casimir antisymmetry conditions . This means that in the linear approximation, the phenomenological laws of energy transformation take the form:
Unlike (6), these laws reflect a decrease in the flow of the primary energy carrier as the overcome force increases and approaches the "idle" mode. Therefore, it is these equations, and not the relations (6) postulated by L. Onsager, that should be called phenomenological (i.e., based on experience) laws.
Let us consider, as an example, an element of a muscle - a fibril, which has the ability to contract when a chemical reaction starts, that is, it converts chemical energy into mechanical energy. In accordance with this, we will take the flow of substances participating in a given chemical reaction as the flow of the primary energy carrier , and the rate of muscle contraction as the second flow . Each of these flows, in accordance with (19) and (20), depends on both forces, the first of which in this case is the negative gradient of the chemical affinity of the reaction - , and the other is the contraction force of the fibril . Note that in the case when the chemical reaction goes to the end ( ), the force is numerically equal to the standard affinity of the chemical reaction . Since chemical reactions are usually described as scalar, in the future we will operate with the modules of forces and flows.
It is more convenient to represent laws (19) and (20) in a dimensionless form that does not contain phenomenological coefficients. For example, consider the regime of the so-called "isometric muscle contraction" when , as well as "unloaded muscle contraction" when . Expressing and in terms of phenomenological coefficients (assuming their constancy), we find under conditions of constancy of forces :
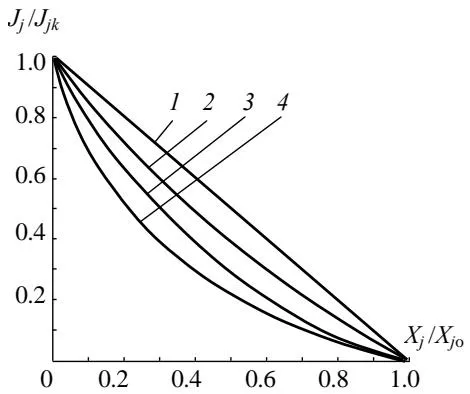
To confirm the applicability of these equations to biological systems, we will use the experimentally found kinetic Hill equations, which quite accurately describe the characteristics of muscles taken from various animal species [5]. The load characteristics of the muscle propellers built on their basis are shown in Figure 2.
Curves 1, 2, 3, 4 in this figure correspond to different degrees of nonlinearity of Hill's kinetic equations. This nonlinearity is usually explained by the relationship between the rates of both processes (flows and ) [4]. In linear systems, the dependence of on in linear systems is expressed by a straight line intersecting the ordinate axes at and (curve 1). It is easy to see that it is precisely this character that follows from the kinetic laws (15). Consequently, the work of the muscle and its element, the fibril, obeys the universal laws of energy dynamics, and the modes of isometric muscle contraction and its unloaded contraction are similar to the modes of short circuiting and no-load and of a motor or a welding transformer.
Thus, the unity of the laws of energy transformation in technical and biological systems is revealed, which makes it possible to transfer the research results of some of them to others. At the same time, another reason for the inapplicability of consumer goods to biological energy converters is revealed. It consists in the fact that when forces and flows are found on the basis of expression (1) TIP, a limitation of the magnitude of their relative efficiency (less than ) arises, which is not characteristic of real energy converters (less than ) [37]. This limitation, however, is absent in the case of antisymmetric reciprocity relations. This confirms once again the inadmissibility of the formal transfer of the known provisions of the theory of irreversible processes to systems that perform useful work.
The independence of Eq. (21) from the structure and size of fibillae allows the theory of the similarity of muscle movers, similar to that for power plants [37]. This theory makes it possible to form a number of dimensionless criteria for the similarity of such systems. One of them, the "design criterion" , is analogous to the ratio of reactive and active resistances, known in radio engineering as the -factor of the circuit, and coincides (up to a temperature factor) with the "Q-factor" , introduced A. Ioffe as a generalizing characteristic of thermoelectric generators (TEG). Its value fluctuates from zero to infinity , increasing with a decrease in "active" resistances (from the side of dissipation forces) and and an increase in "reactive" resistances (from the side of the useful load). Like thermal resistances in the theory of heat transfer, these resistances depend on the properties of muscle tissues and their section, composition, etc.
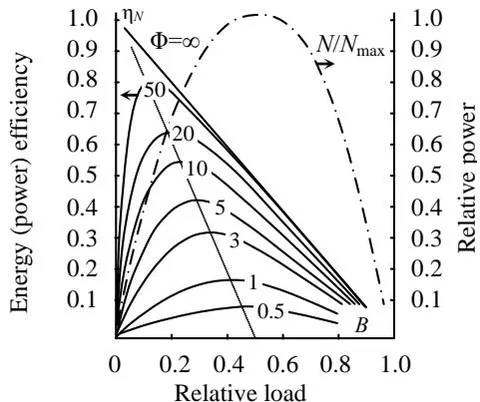
Another dimensionless criterion , called the "relative load", is composed of the boundary conditions specified by the value of the forces or flows . It changes from zero in the "idle" mode ("unloaded muscle contraction) to one in the "short circuit "mode . Using these criteria, expression (23) can be given the form of a criterion equation for the energy conversion process:
Here is the efficiency of the process, expressed by the ratio of the output and the input power, and therefore we called it power. It generalizes the concept of relative efficiency in classical thermodynamics. This efficiency complements the well-known concept of taking into account the kinetics of the energy conversion process and therefore most fully reflects the perfection of the converter, that is, the degree to which it realizes the possibilities that nature provides.
The criterion equation (22) allows constructing a universal load characteristic expressing the dependence of this efficiency on the power and load , as well as the perfection of the energy converter (Figure 3) [37]. The solid lines on it show the dependence of the efficiency on the load criterion at various values of the quality factor , and the dash-dotted line shows the dependence on the load of its output power . As follows from the figure, the efficiency of any power plant vanishes twice: at idle ( ) and in the "short circuit" mode ( ). In this case, the loads corresponding to the maximum efficiency and maximum power diverge the more noticeably, the more perfect the muscular mover. In the absence of any energy losses (from friction, heat release, all kinds of "leaks" of reagents, losses at idle run of the installation, etc., i.e., at ), the power efficiency of the installation increases linearly with decreasing load, and at reaches, as expected, unity. This case corresponds to the ideal Carnot machine, which has the highest thermodynamic efficiency. However, the power of the converter in this mode approaches zero. This indicates the existence of an optimum in terms of efficiency. A mode similar to the nominal mode of the power plant. The versatile features make it easy to find such a compromise. Thus, one more step is taken towards the approximation of the results of the theoretical analysis of the converter to reality.
VIII. THE PRINCIPLE OF SURVIVAL" AS THE BASIC LAW OF THE EVOLUTION OF BIOSYSTEMS
Let us apply the basic identity of energy dynamics (3) to the processes of evolution of biosystems. Introducing the missing nonequilibrium parameters and into it allows us to obtain a number of nontrivial consequences for them [38]. One of them is the conclusion that after the isolation of the nonequilibrium system the processes of energy interconversion, obeying the condition
Let us now take into account that a change in any parameter can be caused not only by relaxation of the -th degree of freedom, but also by the performance of external and internal work by forces and . This circumstance can be expressed by the balance equations of the quantity , similar to the equations of entropy balance proposed by I. Prigogine:
where are the components of the total change in the parameter , caused by the performance of external , internal and dissipative work, respectively.
Accordingly, the flow as the generalized speed of any -th process includes external , reversible internal and dissipative internal components:
In this case, condition (24) in isolated systems takes the form:
According to this expression, as long as relaxation processes are going on in the system , oppositely directed (anti-dissipative) processes of doing internal work "against equilibrium" will also take place in it. In energetodynamics, this position is called the "principle of counter-directionality" of non-equilibrium processes, which can be regarded as a mathematical expressin this case, this principle means that the approach to equilibrium of some degrees of freedom of the system is accompanied by the distance from it of other, -th degrees of freedom . Hence follows the unity of the processes of evolution (complication) and involution (degradation) of nonequilibrium systems. Unlike classical thermodynamics, which cannot say anything about the rate of approach of a biosystem to equilibrium, energy dynamics allows us to raise the question of the rate of approach of the system to a state of equilibrium and the effect of the complexity of a biosystem and its remoteness from a state of equilibrium on the duration of its life. According to(3), under comparable conditions, the rate of relaxation of the system prescribed by the 2nd law of thermodynamics depends on the rate of reversible processes, with the necessity arising in it due to the principle of oppositely directed nonequilibrium processes. In this case, it is of undoubted interest to compare the speed of approaching equilibrium of two arbitrary biosystems of different complexity (with a different number of degrees of freedom).
If, in an arbitrary system, we somehow "freeze" chemical or any other processes associated with the performance of reversible internal work (that is, to direct to zero), then the speed of its approach to equilibrium will become equal to
Comparing (23) and (26), we find that their ratio is determined by the expression:
It is easy to see that this ratio can be either greater or less than one, depending on the sign of the sum , since is always positive. If , that is, there is work "against equilibrium" (and forces ) in the system, then the speed of approach of such a system to equilibrium decreases in comparison with a system where such processes are absent:
and can become equal to zero when work "against equilibrium" becomes equal to work of a dissipative nature. This case corresponds to the onset of a stationary state. Among the macroprocesses in which such counter-directional changes of state take place is the so-called "active transport" of substances, which leads to the accumulation of reagents with a relatively high Gibbs energy in the corresponding organs. The same are the already mentioned processes of "ascending diffusion" in alloys, as well as the so-called "conjugate chemical reactions". Some of them, like the Belousov-Zhabotinsky cyclical reactions ("chemical clocks") or the process of the circulation of matter in the Universe, can continue indefinitely. All processes of this kind require a certain organization of the system and therefore arise only at a certain stage of their evolution. The life span of biosystems, as well as their reproductive period, depends on their intensity, which affects the evolution of the entire subsequent population of this type of bioorganisms.
Here lies the key to understanding the general direction of the evolution of a biological system, understood as a transition from simple to complex. This direction of evolution is not something imposed by the "higher mind" or Darwinian "struggle for existence" - it is a consequence of purely physical reasons reflected in the energodynamic principle of "opposite direction" of nonequilibrium processes. Such are any processes leading to the ordering of the system, the acquisition of new properties by it (an increase in the number of degrees of freedom), the complication of the structure, etc.
At the same time, the "postponement" of the onset of equilibrium in biosystems, achieved due to the occurrence of reversible processes in them, is so close to the Darwinian idea of "struggle for existence" that it can also be called the "principle of survival" for clarity. This principle can be formulated briefly in the form of a statement: "Evolutionary processes occurring in biological systems are directed towards increasing the duration of their life." This provision is so general that it can be considered the basic law of biological evolution.
This law does not at all contradict classical thermodynamics and its second principle, which removes their "flagrant contradiction" noted by I. Prigogine. At the same time, he debunks the myth of "the emergence of order from chaos" [20], since it becomes clear that maintaining "order" requires the expenditure of work, the absence of which in isolated systems is inevitably accompanied by a decrease in their ordered energy. In other words, "order" in any part of the system (subsystem) arises not from ha-os, but due to a higher order in other parts of the system or in the surrounding force fields. For biological systems, these are radiation fields, flora and fauna, which have ordered forms of energy. This radically changes our worldview.
IX. ENERGODYNAMICS AND DARWINIAN THEORY OF EVOLUTION
Let us now show that the well-known "triad" of Darwin's doctrine of evolution [] - adaptability, variability and heredity - are a consequence of the above formulated energy-dynamic law of evolution. Considering biological objects as non-equilibrium systems immersed in a nonequilibrium environment, energy dynamics deepens our understanding of equilibrium. It is one thing when both the system and the environment are homogeneous (that is, they lack both long-range and short-range force fields). Then their equilibrium corresponds to the termination of processes both in the environment and in the system. The condition for such external equilibrium is the equality of the corresponding potential (temperature, pressure, chemical, electrical, etc. potentials) in all parts of the system and the environment. The resulting forces in this case are equal to zero, which corresponds to inaction. It is with this kind of external equilibrium that classical thermodynamics deals. However, the concept of force was alien to classical thermodynamics. Therefore, she distorted the meaning of the concept of equilibrium as an equal action of forces, replacing it with inaction (the absence of any processes).
A different kind of state occurs when both the system and the environment are heterogeneous and the thermodynamic forces in them are nonzero. Then the external equilibrium means their equal action, which does not exclude the occurrence of internal processes in the system and in the environment. Thus, external balance does not at all mean the presence of complete (external and internal) balance. It is with this case that the thermodynamics of biological and ecological processes deals. Equilibrium establishment processes of this kind are adiabatic and therefore do not obey the entropic criteria of evolution and equilibrium. Meanwhile, it is these processes that are responsible for the evolution of biological systems in the direction of establishing a balance between them and the environment. This is Darwinian adaptability in its energy-dynamic understanding. In the course of such processes, the body acquires new properties (new degrees of freedom), which were absent in it in a state of internal balance. The lack of equilibrium with the environment is manifested in the presence of thermodynamic forces , which generate a change in the state of both the system and its environment. This is the thermodynamic reason for the variability of organisms. The result of this process is the equality of the forces in the system and the environment, and not their internal balance. Striving for such a balance by no means deprives the biosystem of the ability to perform useful external work and to internal interconversion of energy.
As follows from the principle of survival, partial equilibrium lengthens the time the system remains in a nonequilibrium state. Then, in the presence of inevitable mutations of the hereditary code, the degree of their probability increases. Thus, better "adapted" individuals acquire an advantage in the transmission of gene information. This is the energy-dynamic nature of heredity. It is characteristic that all three named basic provisions of the Darwinian doctrine of evolution turn out to be a consequence of a single criterion of "survival" - the minimum speed of the system approaching equilibrium.
In the "theory of neutrality" of evolution (L. Blumenfeld, 1977), energetodynamics can explain the mechanism of elimination (preservation of random genetic changes), since the probability of this process from the standpoint of the "principle of survival" increases with the lengthening of the life of a better adapted (closer to external equilibrium) individual. In the theory of "jump-like evolution" ("punctualism"), energy dynamics can explain the jump-like increase in the rate of change of genes, since it recognizes the inevitability of "bifurcation" (branching of process trajectories) with distance from equilibrium. In the theory of "molecular evolution", energy dynamics is able to explain the change in the composition of living organisms in ontogenesis, since natural aging is accompanied by a decrease in their specific energy. Thus, energetodynamics can serve as a touchstone for any of the evolutionary theories.
X. CONCLUSION
The reason for the "glaring contradiction" between equilibrium thermodynamics and the theory of biological evolution is the absence in its equations of time as a physical parameter and its inability to take into account the kinetics of real processes. This contradiction persists in the theory of irreversible processes, which excluded from consideration the reversible part of such processes.
Description of the state of nonequilibrium systems requires the introduction of intense and extensive parameters of spatial in homogeneity, characterizing their deviation from equilibrium. These parameters have a number of advantages over entropy, reflecting the approach to equilibrium and the distance from it both for the system as a whole and for each of its inherent degrees of freedom separately.
The introduction of these parameters of spatial heterogeneity into thermodynamics reveals the occurrence in nonequilibrium systems of reversible processes of redistribution of energy carriers over the volume of the system and their opposite direction, reflecting the dialectical unity of opposites.
The use of these parameters and as criteria for their evolution and involution reveals the inevitability of the simultaneous occurrence of these processes in different parts (regions, phases and components) of the nonequilibrium system and the interconversion of energy in them, accompanied not only by its relaxation, but and doing work "against equilibrium."
The processes of performing external and internal work in the muscle tissues of living organisms are subject to the same laws as the processes of energy conversion in various thermal and nonthermal machines. This makes it possible to create a theory of the similarity of muscular energy converters, which facilitates the selection of the optimal modes of their activity.
The course of oppositely directed processes in biological systems slows down their approach to equilibrium and makes it possible to formulate the "principle of their survival", according to which their self-organization leads to an increase in the duration