I. INTRODUCTION
Riparian ecosystem fluxes are a function of the pulsations of the water cycle mainly controlled by climate and anthropogenic perturbations. The increasing pressure on these ecosystems for provision of goods and services in the century and beyond coupled with increasing sensitivity to climate change poses a threat to their sustainability (Capon et al., 2013, Maxwell et al., 2016). Isolated evidence in the literature is suggestive of a likelihood of acquired resilience of these systems to climate change due to exposure to extreme conditions of environmental variability (Capon et al., 2013). There is consensus among scholars that management adaptation and mitigation strategies are critical in the quest to reduce vulnerability and enhance capacity for adaptation to changing environmental and extreme hydrological conditions (Hulme, 2005, Palmer et al., 2007 and Steffen et al., 2009).
There is no doubt that riparian ecosystems at various spatial and temporal scales influence flow of energy and material cycling between and within connected terrestrial and aquatic ecosystems. The ecological significance of energy transfer and material cycling in the performance of trophic systems associated with trophic level interactions, food webs and food chains as well as provisional services for supporting human livelihoods cannot be overemphasized. At the abiotic level, riparian functions have considerable influence on the carbon and nitrogen sequestration, hydrologic and geomorphological processes, sulphur and phosphorous cycles as well as biogeochemical cycles and other processes in landscapes. Integrated biotic and abiotic interactions at larger scales of riparian ecosystem functions regulate climate, biodiversity, hydrologic processes, nutrients, soils, and autotrophic and heterotrophic level performance (Sala et al.,2000, Habel and Ulrich, 2021). Non-disturbed ecosystems with rich biodiversity have been demonstrated to effectively and efficiently offer ecosystem functions compared to degraded and homogenous ecosystems (Winqvist et al., 2011). Anthropogenic activities erode ecosystem functions. Overgrazing, deforestation as well as selective extraction of plant materials from riparian ecosystems influence hydrologic processes that cause microclimatic modification with significant consequences on water and energy budgets (Lawrence and Vandecar, 2015, Felipe-Lucia et al., 2020). Introduction of invasive exotic species with the potential of hybridization and adulteration of indigenous plant material genetic pools reduce the diversity of ecosystem functions on offer (Linderset al., 2019, Baude et al., 2019).
The diversity of riparian ecosystem functions provides a super structural base for human development through extraction of primary resources in the form of goods and benefit from services as well as a support system for other abiotic- biotic interactions that provide synergies for physiological and ecological processes (Millennium Ecosystem Assessment, 2005, Klein et al., 2007, Power, 2010 and Tschumi et al., 2018).
Subsistence farmers dependent on livestock products and limited non-rainfed horticultural production serviced by coastal riparian ecosystem functions for their livelihood must continue to contend with a high food security risk in the absence of successful adaptation and mitigation efforts to reduce vulnerability to environmental variability and climate change (Hulme, 2005). This scenario is predicated by inappropriate land use systems, increasing demographic pressure as well as weak infrastructural frameworks for the management and governance of riparian ecosystems.
The need for adaptation options and mitigation efforts anchored on baseline ecological and socioeconomic profiles for conservation of dynamic and rapidly degenerating riparian ecosystems provided the motivation for the current study.
Previous research work on riparian ecosystems affirms the fact that there is a general understanding regarding the response of terrestrial and wetland ecosystems to human perturbations, however, there is a dearth of information on the response of riparian ecosystems to ecologic and socio-economic impacts(Sala et al., 2000, Hooper et al., 2005, Power, 2010, Habel et al., 2015, Habel et al., 2018). The primary objective of this paper is to present research evidence on the response of River Lumi riparian ecosystem to ecologic and socio-economic impacts and contextualize management implications for arresting biodiversity loss.
II. MATERIALS AND METHODS
a) Description of Study Area
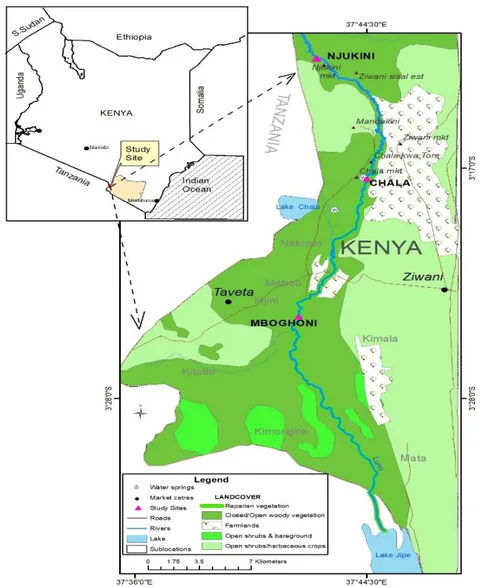
The source of River Lumi is Mt. Kilimanjaro. The river flows north eastwards traversing a water catchment rich in riparian vegetation, closed and open wood vegetation and open shrubs before crossing the border from Tanzania to Kenya and draining into Lake Jipe in Taita Taveta County (Figure 1). River Lumi riparian ecosystem with an area of provides goods and services for the communities that have settled along the river(Ngugi et al., 2015). These include irrigation water, timber and grass for house construction as well as firewood for supply of energy for cooking and other purposes. The river ecosystem provides a life support system for wildlife in the adjacent Tsavo East and West National Parks.
b) Topography and Climate
The study area is a dissected lava plateau with half dozen isolated hills south of Taveta and Mt. Kilimanjaro volcanic pile. The tertiary lavas of Mt. Kilimanjaro volcanic pile consist of Rombo series with manifestations of Kijabe type basalts, olivine basalts and olivine soda trachytes. River Lumi watershed area exhibits topographical variations ranging between 1200 meters above sea level (m.a.s.l) and 1800m.a.s.l. There are innumerable small volcanic cones represented by Kijabe basalt. Projecting above the landscape, between Lake Chala and Lake Jipe are pyroclastic cones contaminated with olivine basalts.
The climate of River Lumi riparian ecosystem is characterized as semi-arid area receiving a mean annual rainfall of 616mm. Mean monthly maximum temperature is of the order of and a mean monthly minimum of (Republic of Kenya, 2014).
c) Geology and Drainage
The geology of the River Lumi water catchment consists of parent metamorphic rocks that have disintegrated by weathering and geomorphological processes into sedimentary alluvium and deposited by several streams that feed into River Lumi before it drains into Lake Jipe. Substantial superficial deposits on the flood plain include calcareous and ferruginous clays and white gritty and greyish limestone with carbonaceous material of fluvio-lacustrine origin(Bear, 1955, Horkel, et al., 1979: Geology of Taita Hills Quadrangle; with a geological map 1:50.000, Kenya).
River Lumi cuts deeply across the grain of the basement rocks and is fed by several springs at the junction of Njoro Kubwa before it empties into Lake Jipe. The ruggedly eroded channel is approximately 4metres deep and is characterized by heavy deposition of alluvium and sedentary soils of metamorphic origin in the lower reaches of the river. The bed of the channel is mainly basalt. The river is prone to considerable flooding and materially destructive to road and railway infrastructure as well as irrigation projects in its flood plain. There are traces of effects of tertiary volcanity that may have deflected Lumi streams that flowed into the Tsavo to the east of Sambera where the watershed between Lumi and Njoro is less than 100 metres (Horkel et al., 1979).
d) Biodiversity
River Lumi ecosystem has diverse flora and fauna. The natural vegetation type is savannah grassland with scattered Acacia trees, bushes and semi-arid shrubs. Belts of evergreen riverine vegetation occur particularly in the fringes of the flood plain. Dominant tree species include Tabernaemontana stapfiana, Pauridiantha clauracea and Acacia nubica (Wekesa et al., 2018). The riparian ecosystem provides a life-support system for the rich fauna including a variety of water birds, zebras, elephants, impalas and gazelles in the Tsavo West National Park. River Lumi flood plain is an extensive area supporting irrigation agriculture. The dry savannah is an important grazing area for livestock.
e) Settlement and Land Uses
The communities that have settled along River Lumi watershed carry out subsistence crop and livestock farming with limited commercial irrigated farming (Muli, 2014). According to KNBS, 2019, a population of 9122 are dependent on small business enterprises in the major trading centres in the riparian ecosystem. These enterprises revolve around livestock and crop products and mainly horticultural products, timber craft wares, as well as fishing within Lake Jipe. River Lumi riparian ecosystem and its proximal areas have a large proportion of squatters whose livelihood activities have contributed significantly to degradation of the ecosystem (Ngugi et al., 2015).
f) Socio-economic Profiles
Economic production systems based on land uses were identified and categorized into three socioeconomic profiles. The upper reaches of River Lumi ecosystem represented by Njukini location is a livestock grazing area mainly used by the Maasai community. A large number of livestock are kept on private ranches on the river Lumi water catchment. There is also a considerable density of medium scale livestock subsistence farming to cater for the livelihood requirements of the communities in the water shed area. The middle zone represented by Chala location is a mixed crop-livestock area mainly used by the Kamba community. The lower reaches of River Lumi represented by Mboghoni is a predominantly crop farming area utilized by the Taita Taveta community. Commercial horticultural crops based on irrigation systems such as tomatoes, cabbages, kales, capsicum are grown. Other crops include bananas and maize (Muli, 2014, Ngugi et al., 2015 and Njiriri, 2016). There are scattered small business enterprises as well as fishing mainly in Lake Jipe to complement the income sources of the community settled in the riparian ecosystem (Njiriri, 2016).
III. ENVIRONMENTAL AND SOCIOECONOMIC DATA
Exploratory socio-economic surveys as well as vegetation measurements were carried out. Semi-structured household questionnaires and Focus Group Discussions (FGD) were designed to obtain data on the interaction between socio-economic factors comprising demographic change, gender, income and education levels, land size relegated to crops and livestock, commodity prices and household response to the degradation of River Lumi ecosystem. Field assessments of forest structure, tree species diversity and soil characteristics that influence tree species type and distribution in Njukini, Chala and Mboghoni locations yielded the data requirements of this study.
a) Vegetation Data
Tree height and diameter at breast height (DBH), species richness, species diversity and regeneration were determined in plots and sub-plots along 36 belt transects. The plots measured by 15.0 whereas the sub-plots were by . The plots were established with the long side perpendicular to the river bank.
A diameter tape was used to measure DBH of trees greater than . Nested sub-plots within main plots measuring by and by were used for measurements of saplings and seedlings. Saplings were designated as trees with DBH whereas seedlings were defined as trees with DBH .
Tree species diversity was estimated using Shannon-Weiner diversity index(Shannon and Weaver, 1963; Krebs, 1999), whereas species richness was determined by counting different tree species found in the plots. Shannon-Weiner index is a measure of species diversity in a community and accounts for species abundance and evenness. Typically, Shannon diversity index values range between 1.5 and 3.5 and rarely exceed 4.0 in most ecological studies. Usually, values less than 1.5 signify low diversity, values between 1.5 and 2.5 indicate medium diversity and values greater than 2.5 represent high diversity.
Shannon-Weiner index is defined as:
Where,
H = Species diversity index
Proportion of individuals of each species belonging to the ith species of the total number of individuals
S= Number of species in the community
Species richness and diversity was compared in the three land use systems (livestock production, mixed farming and crop farming) along River Lumi riparian ecosystem.
b) Soil-vegetation Interaction Data
Soil samples were collected from Njukini, Chala and Mboghoni locations in July 2019 and 2020 for determinations of soil pH, organic carbon, nitrogen, phosphorous, potassium and soil moisture content. Soil augers were used to collect three replicates of soil samples from 0-15cm and 15-30cm soil depths within the sub-plots in the 36 belt transects where vegetation measurements were carried out. A total of 300 composited soil samples were analyzed at the Kenya Forestry Research Soil Science Laboratory in Muguga, Kenya.
Samples were air dried and sieved using sieve prior to analysis. Soil moisture content was gravimetrically determined using Okalebo et al., 2002 procedure. Olsen and Kjeldahl methods were used in the determination of nitrogen and phosphorous (Okalebo et al., 2002). The Walkley-Black method was used in the determination of organic carbon through complete oxidation (Walkley and Black, 1934). Potassium was determined using Kjeldahl procedures and photometric analysis using a photoelectric flame photometer(Okalebo et al., 2002). Soil pH was measured using a pH meter as described by Anderson and Ingram 1993. Soil pH, soil moisture content and soil chemical composition were used in providing plausible explanations for the variation and distribution of tree species along River Lumi riparian ecosystem.
The measure of association between the distribution of tree species and soil chemical characteristics in the upper, middle and lower reaches of River Lumi was determined by Canonical Correspondence Analysis (Wekesa, 2018). Tree species were classified into dominant, less dominant and rare categories where the proportion of occurrence in the sampled plots was at least , less than and respectively.
An estimate of species heterogeneity was obtained through detrended corresponding analysis (DCA) prior to Canonical Correspondence analysis (CCA). Preliminary DCA test revealed that the tree species interactions exhibited unimodal responses of six standard deviations (SD), making CCA the most appropriate method for analysis (Leps and Smilauer, 2003). The association between soil characteristics and tree species distribution as well as the relationship between dominant tree species, less dominant and rare species along River Lumi riparian ecosystem was determined by the application of CCA with automatic forward selection using 1000 permutations at probability level and verified by Monte-Carlo Permutation Test (MCPT).
c) Socio-economic Data
Socioeconomic data was obtained from three stratified administrative units within Njukini, Chala and Mboghoni locations using systematic sampling procedures. These administrative units comprised Njukini springs-Chala Kwa Tom in the upper reaches of River Lumire presenting the livestock production system, Madulu springs-Darajaniiin the middle zone was representative of the mixed farming system whereas Njoroya Katembo-Mboghoni in the lower reaches of
River Lumire presented the crop production system. The households with settlements approximately five kilometers from River Lumire were systematically sampled in proportion to the total number of households in each location. The estimated number of households in Njukini, Chala and Mboghoni was 2,295, 1,325, and 790 respectively (KNBS, 2010). Thus 184, 105 and 64 households representing at least (Mugenda and Mugenda, 1999) of the households living in Njukini, Chala and Mboghoni locations were selected and interviewed using semi-structured questionnaires. A total of 353 respondents were interviewed.
The 2009 Kenya National Bureau of Statistics Household Census data for the selected locations (Njukini, Chala and Mboghoni) was used in determining the sample size. The three study locations have 4,410 households (KNBS, 2010). The sample size for the households was calculated using the following formulae recommended for population size of less than 10,000 (Cochran, 1963).
N
where is desired sample size when population is less than 10,000
is the desired sample size
N is the estimated population of the three locations
Therefore, the total sample size for the 3 locations was,
This figure (353) was distributed in the three locations proportionately based on total number of households as shown in Table 1.
| Location | Total number of households | Sample size (nf) |
| Njukini | 2,295 | 184 |
| Chala | 1,325 | 105 |
| Mboghoni | 790 | 64 |
| Total | 4,410 | 353 |
Focus Group Discussions (FGDs) and semi-structured questionnaires were used in the collection of primary household data. Secondary data regarding population profiles, levels of education, land sizes relegated to different land use systems, income level, gender, household size and market dynamics was obtained from Kenya Government Departments as well as Kenya National Bureau of Statistics. A total of 35 questionnaires comprising of the sample projected for the larger parent study (Connelly, 2008) was used in the pilot survey. Pilot surveys for pretesting the research instrument for validity and reliability were conducted in Nakuruto village adjacent to Chala location in the middle zone of the riparian ecosystem. The focus of sample survey revolved around the land resource ownership, livelihood activities and their consequences on the dynamics of the integrated resources of the watershed, water resources governance and community participation in the conservation of riparian resources. Current and historical drivers of riparian degradation were constructed through discussion discourses (FGDs) involving mixed-crop production systems, crop production and livestock production systems in the three study locations. Government and non-Governmental key informants as well as community-based organizations (CBOs) were involved in interactive discourses to provide and verify information on the significance of socio-economic factors on the dynamics of the riparian ecosystem.
d) Data Analysis
Prior to data analysis, normality and reliability attributes were tested using Cronbach alpha reliability function for socioeconomic data and Levene's test for ecological data respectively. Square root transformation of count data on the number of tree species per plot for each observation was performed to correct nonnormality before parametric analysis. Parametric statistics were used to analyze tree species diversity, stand density, species richness, diameter of trees at breast height and height as well as household income.
Tukey's post hoc test with a probability significance threshold was used to separate least significance difference in means. The F-test isolated significant effects associated with the independent variables at confidence interval. The association between land tenure, education level, income level, gender, household size and house hold response to degradation through participation in conservation activities was evaluated by means of Spearman's rank correlation analysis.
IV. RESULTS AND DISCUSSION
a) Vegetation dynamics in the contrasting livestock, mixed farming and crop production systems
Natural regeneration plays an important role in forest succession and enhances tree species diversity. Tree species regeneration along the riverine ecosystem was studied in the context of varying land production systems. The seedling density was higher in the crop production system (461.77±255.16 stems/ha), as compared to livestock production system (400.20±169.57 stems/ha), and mixed farming system (387.62±64.44 stems/ha) (Figure 2). The seedlings density in the three land use systems was, however, not significantly different (F (1, 2) = 0.07; p=0.937). Similarly, the sapling density in the three land use systems was not significantly different (F (1, 2) = 0.44; p=0.647), although the saplings density was higher in crop farming system (385.23±74.49 stems/ha) than mixed farming system (302.58±37.76 stems/ha) and livestock production system (293.64±59.75 stems/ha). A similar trend was observed in shrubs density (stems/ha). The shrubs stand density in the three land use systems was not significantly different (F (1, 2) = 0.77; p=0.471), although higher shrub density was recorded in mixed farming system (1037.56±255.01) than in livestock production system (799.20±274.78) and crop farming system (448.44±153.87).
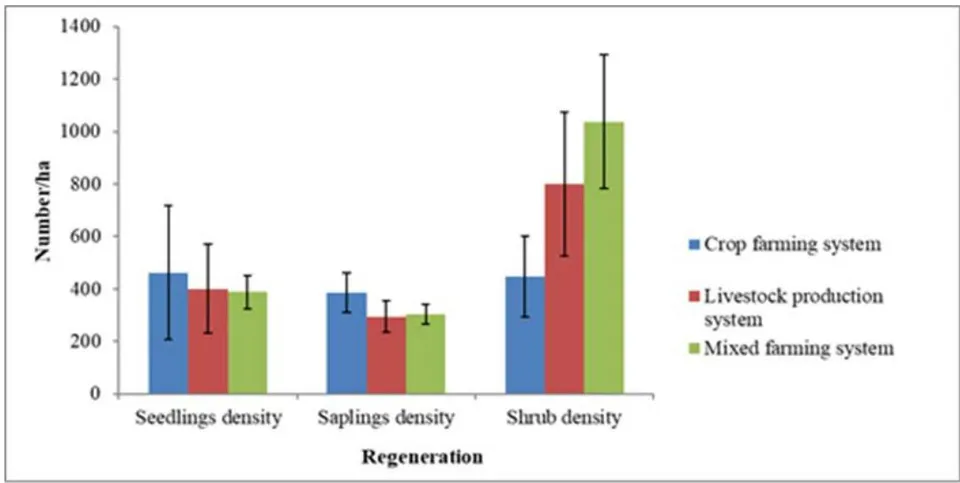
The effect of land production system on natural regeneration was evident in the three land use systems.
Both seedling and sapling densities were higher in crop farming system than in mixed farming system and livestock production system. Mixed farming and livestock production systems had negative impacts on natural regeneration. The low seedlings and saplings density in the livestock production system was attributed to browsing and trampling by animals as well as soil compaction which inhibits seedlings and saplings growth. These results are in conformity with the intermediate disturbance hypothesis (IDH) which predicts the behaviour of species diversity under different disturbance levels in stream ecosystems (Connell, 1978). According to IDH, moderately disturbed areas record high species diversity due to the low magnitude and frequency of disturbances which have a minimal effect on plant communities. On the contrary, areas with more frequent and intense disturbance often have low species diversity since species that regenerate quickly between disturbance events will prevail. In this study, the crop farming system was characterized by moderate disturbance while the livestock production and mixed farming system were characterized with heavy disturbance. The heavy disturbance due to overgrazing in the livestock production system as well as the multiple land uses (crop farming and livestock production) in the mixed farming system could explain the low natural regeneration in the two land use systems. Evidence from previous studies shows that intense land use such as overgrazing impedes forest recovery. This is mainly due to high prevalence of grasses and other herbaceous species which inhibit the establishment of woody vegetation (Zahawi and Augspurger, 1999; Kennard, 2002; and Makana and Thomas, 2006).
The crop farming system had adequate light in the understory, and had higher species diversity which provided a seed source to facilitate tree seedling growth (Nostrand et al., 2003). In Mboghoni location, the crop farming zone experienced wet environmental conditions facilitating seed germination and seedling growth as compared to Chala (the mixed farming zone) and Njukini (livestock production zones) which are situated in arid and semi-arid lands (ASALS) (Republic of Kenya, 2018). Dry conditions slow litter decomposition (Didham, 1998) and accumulating litter may affect seed germination and seedling survival negatively (Bruna, 1999; Wekesa, 2018). River Lumi flood plain where the crop farming system is practiced receives deposits of alluvial soils along the river bank enhancing the nutrient levels which facilitate growth of seedlings and saplings. High soil moisture content resulting from irrigated farming and alluvial soil deposits in the crop farming system also provided favourable environmental conditions for seedling growth. These findings are in agreement with previous studies that have corroborated evidence that site-specific factors such as soil type and nutrient availability, soil pH, moisture, sunlight, microtopography and competition have an effect on species regeneration and growth (Nostrand et al., 2003; Wekesa et al., 2018). As expected, shrub density was marginally higher in mixed farming system and livestock production system than in crop farming system. The low seedling and sapling densities in mixed farming and livestock production systems were attributed to high shrub density. Dwire et al., (2018) who assessed the effects of climate change on riparian areas in the Blue Mountains in Oregon, USA established that reduced soil moisture resulting from drought and dry weather conditions often leads to increase in non-native species and transition from riparian woody plants to drought tolerant conifers and shrubs. The results of this study imply that climate change may have influenced the low seedling and sapling densities in the mixed farming and livestock production systems which are vulnerable to extreme climatic conditions due to their location in semi-arid areas. According to Adel et al., (2018), an increase in shrub density in riparian areas intensifies competition for light and nutrients between tree seedlings and shrubs leading to reduction in seedling density. Additionally, shading from shrubs reduces tree seedling density. Hudson et al., (2014) observed that the shading effect of shrubs along riverbanks reduced seedling density and tree regeneration, while Sarr et al., (2011) noted that high shrub densities in riparian forests caused out-competition of seedlings leading to low seedlings densities and regeneration.
There were higher densities of shrubs in both crop-livestock system and livestock production system. The shifts in botanical composition arising from differential livestock utilization has been demonstrated by Ratovonamana et al., (2013). In their study, they found that changes in the structure of woody plant species resulting from browsing favours the growth of herbaceous and unpalatable species. On the basis of this evidence, it can be surmised that the higher densities of shrubs in both mixed farming system and livestock production system may be attributed to differential utilization by livestock. Ratovonamana et al., (2013) also found evidence that regeneration potential in livestock production zones depends on the browsing intensity and grazing pressure (Reed and Clokie, 2001; Sassenand Sheil, 2013) indicating that intensive grazing hampers forest regeneration. Thus, there is need to ensure appropriate stocking levels that will reduce the grazing pressure particularly in the livestock production system. The complex interactions between land use and land cover in human-dominated landscapes interfere with biotic and abiotic factors and processes, with negative impacts on wildlife habitats, species diversity and abundance, as well as distributional ranges of species (Sala et al., 2000). For instance, forest regeneration in tropical landscapes is often hindered by disturbance in most agricultural landscapes resulting from soil compaction, nutrient loss, and low seedling availability (Ferraz et al., 2005; De Paula, 2018). According to Malik and Bhatt (2016) and Maua et al.,
(2020), the population dynamics of seedlings, saplings and adults tree species can determine the regeneration status of a forest, and effective management of natural forest ecosystems require an understanding of the natural regeneration processes and dynamics.
b) Effect of land production system on forest structure
Stand density and tree sizes are attributes of forest structure that influences the ability of the forest to provide ecosystems goods and services. The mean DBH of trees in the three land use systems was significantly different (F ; . The livestock production system had trees with larger diameters than mixed farming system and crop farming system .
On the contrary, the mean height of trees was not significantly different in the three land use systems (F (1, 2) = 1.35; p=0.259) although the mean height of trees was higher in crop farming system (12.31±1.01) than livestock production system (11.20±1.004) and mixed farming system (10.38±0.628). Similarly, tree stand density in livestock production system, mixed farming system and crop farming system was not significantly different (F (1, 2) = 2.23; p=0.110). The tree stand density was, however, higher in crop farming system (54.95±11.82) than livestock production system (52.60±6.77) and mixed farming system (39.55±3.21), Figure 3.
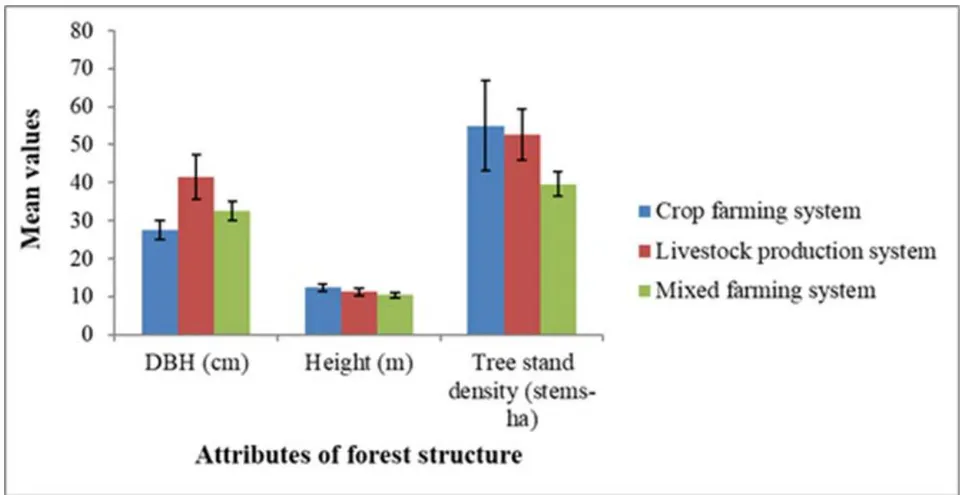
The higher tree stand density in the crop farming system than in livestock production system and mixed farming system may be attributed to high fertility of the soils in the irrigated flood plain frequently enriched by alluvial soil deposits. The fertile riparian flood plain coupled by favourable soil moisture supplies provided a favourable environment for seedling growth leading to higher tree stand density. De Paula (2018) argued that high soil moisture is a precursor to favourable conditions for microbial activity, enhancing decomposition and mobilization of critical mineral nutrients that promote tree growth. Illegal logging and charcoal burning were prevalent in the mixed and livestock production systems. These anthropogenic activities opened up riparian forest areas in Njukini and Chala. Evidence from previous studies also suggests that the low density of trees in Njukini and Chalais due to over-exploitation of such trees through illegal logging and charcoal production among other anthropogenic disturbances (Girma et al., 2014; Maua et al., 2020).
The low tree heights in the mixed farming system were attributed to high demand for crop stakes which are used for supporting tomato crop, a major crop grown in the area. The low mean tree height in mixed farming systems and livestock production systems were further attributed to browsing, trampling and breakages resulting from grazing pressure (Ratovonamana et al., 2013). The livestock production system is dominated with herbaceous vegetation and shrubs which are generally short. Ramirez et al. (2018) has contended that the density and browsing intensity of animals determine the net effect of defoliation on the ecosystem.
Big trees in the crop farming system were cut to attenuate their shade effect on crops. Livestock production in both crop-livestock and livestock production systems had an effect on seedling and sapling density through browsing and trampling hence affecting regeneration, but had no observed effect on mature trees. This explains the higher DBH in the two land use systems.
Previous studies indicate that habitat modification alters ecosystem composition, species distribution and numbers (Stomsand Estes, 1993; Guariguata and Ostertag, 2001), leading to change in ecosystem composition, structure, and functioning (Budowski, 1965; Franklin et al., 2002; Chazdon, 2014). For instance, a study conducted to assess the effect of land use on the structure and diversity of riparian vegetation in the Duero River watershed in Mexico revealed that the land uses adjacent to the riparian area modified attributes of riparian vegetation, particularly species richness and density of stems and individuals (Mendez-Toribio et al., 2014). It was further established that there was a drastic loss of species diversity related to the disturbance generated by the anthropogenic activities ongoing in the vicinity of the river bank.
Evidence from other studies shows that the ecosystem trajectory after a disturbance will depend on the intensity, duration, and frequency of the disturbance, as well as the resilience and stability of the ecosystem (Holling, 1973; Chapin et al., 2011; Clewelland Aronson, 2013). Ecosystems are more likely to bounce back to their pre-disturbance conditions if the disturbance is less severe (Chapin et al., 2011; Hodgson et al., 2015), while in cases of severe disturbance, the ecosystem may shift to an alternative stable state that can persist beyond the disturbance (Holling, 1973; Chapin et al., 2011). The alternative stable state often experiences reduced ecological processes than the previous ecosystem thus sustaining less biodiversity (Clewelland Aronson, 2013). In this study, livestock production system experienced the highest form of disturbance as indicated by the observed land degradation attributed to over-grazing and soil erosion. There is evidence that species composition and vegetation structure significantly changed with increasing grazing pressure. From previous results, it has been established that grazing leads to desertification and soil erosion, resulting in loss of essential nutrients and soil organic matter which support vegetation growth (Guggenberger et al., 1994; Foley et al., 2005).
c) Interaction between soil characteristics and dominant tree species
There was a significant interactive effect between soil physical and chemical characteristics and distribution of five dominant tree species (Vachellia (Acacia) nubica, Ekerbergia capensis, Grewia bicolor, Tabernaemontana stapfiana and Trichilia emetica), and soil physical and chemical characteristics (soil moisture, organic carbon, phosphorous, nitrogen, potassium and pH) along River Lumi riparian ecosystem (F ). The occurrence of dominant tree species was mainly influenced by soil moisture, organic carbon and pH. The occurrence of Ekerbergia capensis was strongly influenced by moisture level in the soil while the occurrence of Grewia bicolor was significantly determined by pH and organic carbon (Figure 4). Occurrence of Tabernaemontana stapfiana and Trichilia emetica was slightly influenced by pH and organic carbon while the occurrence of Vachellia (Acacia) nubica, had no correlation with the soil variables. Nitrogen, phosphorous and potassium did not affect the distribution and abundance of dominant tree species along the riparian forests of River Lumi.
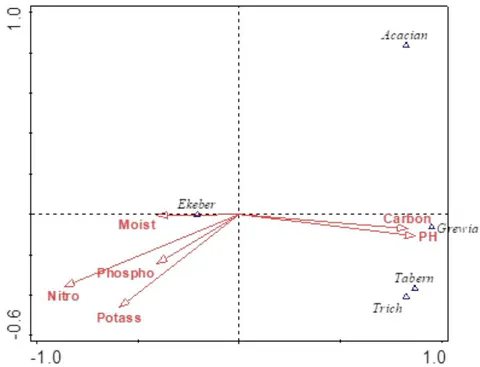
Soil pH, organic carbon, nitrogen and potassium were not significantly different in livestock and mixed production systems. However, phosphorous and soil moisture were significantly different. Soil pH was higher in the livestock production system than in mixed and crop farming systems. Evidence from previous results indicates that irrigated areas in crop and mixed farming systems had higher pH levels than non-irrigated areas where livestock grazing is mainly undertaken(Muli 2014). According to Muli (2014), crop irrigation leads to salinization and affects availability of soil nutrients such as nitrogen, phosphorous and potassium which are easily lost through leaching. High pH recorded in the livestock production system in this study was attributed to the dry conditions in the area while the high acidity found in the crop and mixed farming systems was attributed to the effect of acidifying synthetic fertilizers which were heavily used in the two land use systems. There is evidence that, nitrogen inputs from synthetic fertilizer increases soil acidity in the absence of lime addition (Tarkalson et al., 2006; Liebig et al., 2017). Soil pH has a major influence on the availability of potassium, phosphorus and other nutrients which affect plant growth, hence affecting tree species occurrence and distribution in riparian forests (John et al., 2007).
Phosphorous is frequently excreted via livestock excreta (Wang, 2016) and is thus concentrated in the livestock production system, while continuous harvesting of crops which is mainly practiced in irrigated areas, often depletes phosphorous at a faster rate than natural regeneration (NyanjomandK'Onyango, 2008; Muli, 2014). This is a plausible explanation for lower levels of phosphorous in continuous irrigated crop farming systems. The higher soil moisture content in the crop farming system was attributed to higher rainfall experienced in the crop farming land use system coupled with irrigated farming (Ngugi et al., 2015).
d) Interaction between soil characteristics and less dominant tree species
Soil characteristics were found to influence the distribution of less dominant tree species (F (1000) =2.4; p=0. 01). Occurrence of C. africana, M. excelsa and A. xanthophloeia was strongly influenced by nitrogen content, available phosphorous and soil moisture content. A. abyssinicus had a positive correlation with phosphorous and potassium while A. drepanolobium had a weak positive correlation with potassium (Figure 5). The abundance of F. sur and F. thonningii was slightly influenced by organic carbon, while F. sur, A. melifera, A. abyssinicus and A. drepanolobium had negative relationship with pH.
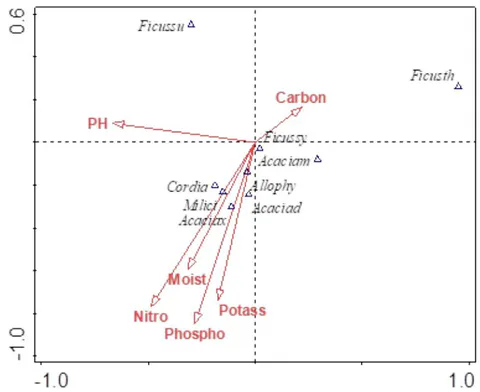
The occurrence of less dominant tree species was mainly influenced by nitrogen, phosphorous and potassium which play a critical role in plant growth
(Omoro et al., 2011), as well as soil pH which affects availability of plant nutrients (John et al., 2007).
e) Interaction between soil characteristics and rare tree species
Environmental variables did not have a major influence on the occurrence and distribution of rare tree species which included (Albizia glaberrima, Albizia gummifera, Bridelia micrantha, Xymalos monospora, Senna denimetria, Senna spectabilis, Croton macrostachyus, Rauvolfia caffra, Ehretia petiolaries, Tapra fisc, and Sorindeia madagascariensis) (F (1000) =2.3; p=0.002). Accordingly, there was no relationship between Albizia glaberrima, Bridelia micrantha, Xymalos monospora, Senna denimetria, Senna spectabilis, Croton macrostachyus, Rauvolfia caffra, Taprafisc, and Sorindeia madagascariensis with any of the soil characteristics studied. Ehretia petiolaries and Albizia gummifera, however, exhibited a strong positive relationship with phosphorous, and a weak relationship with nitrogen and carbon (Figure 6).
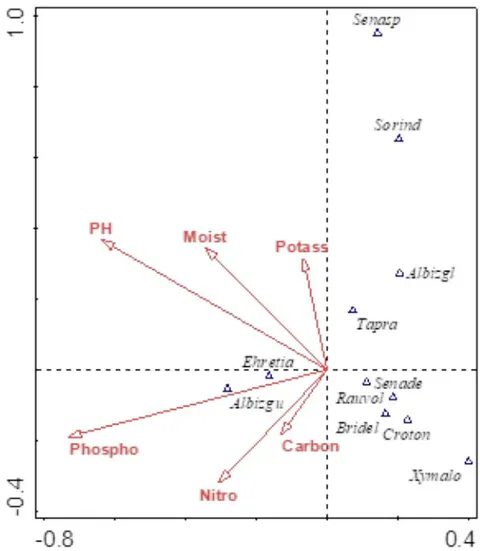
This would suggest that soil variables may not have been entirely responsible for the occurrence and distribution of the rare tree species. Chen et al., (2014), confirmed that external factors such as environmental and ecological conditions, prevalence of human activities and land use type affected the distribution patterns of rare plant species. Similarly, Thammanu et al., (2021) attributed species composition and distribution to a combination of topographic, edaphic, and anthropogenic factors.
f) Interaction between dominant and less dominant tree species along River Lumi riparian ecosystem
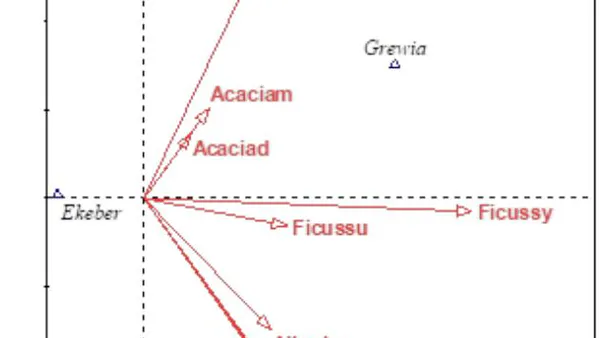
The occurrence of dominant (Vachellia (Acacia) nubica, Ekerbergia capensis, Grewia bicolor, Tabernaemontana stapfiana and Trichilia emetica), with less dominant species (Vachellia (Acacia) drepanolobium, Vachellia (Acacia) mellifera, Vachellia (Acacia) xanthophloeae, Allophyllus abyssinicus, Cordia africana, Ficus thonningii, Ficus sur, Ficus sycomorus and Miliciaexcelsa) was assessed to ascertain their interaction in the natural environment. Canonical Correspondence Analysis (CCA) model was significant for the interaction between dominant and less dominant tree species along River Lumi riparian ecosystem (F .Vachellia (Acacia) nubica and Grewia bicolor had a positive correlation with Ficus thonningii. Similarly, Ekerbergia capensis had a positive correlation with Vachellia (Acacia) mellifera, Vachellia (Acacia) drepanolobium, Ficus sur and Ficus sycomorus. Trichiliaemetica and Tabernaemontana stapfiana had a positive correlation with Allophyllus abyssinicus, Milicia excelsa, Cordia africana and Vachellia (Acacia) xanthophloeae (Figure 7).
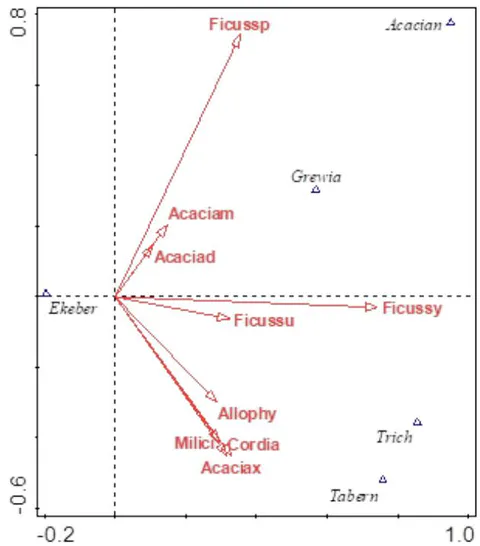
Vachellia (Acacia) nubica, Grewiabicolor andFicus thonningiiwere dominant in the livestock production system. Ekerbergia capensis was a dominant species in themixed farming system and occurred together with Vachellia (Acacia) mellifera, Vachellia (Acacia) drepanolobium, Ficus sur and Ficus sycomorus, while Trichiliaemetica and Tabernaemontana stapfiana had a positive correlation with Allophyllus abyssinicus, Miliciaexcelsa, Cordia africana and Vachellia (Acacia) xanthophloea. The association between Vachellia (Acacia) nubica, Grewia bicolor and Ficus thoningii could be attributed to their tolerance to dry and saline conditions (Sanchez-Bayo and King, 1994)in the livestock production system. These species are also high value fodder trees in the livestock production system (Smith, 1992; Asmare and Mekuriaw, 2019). The association of Ekerbergia capensis, Vachellia (Acacia) mellifera, Vachellia (Acacia) drepanolobium, Ficus sur andFicus sycomoru was attributed to their adaptation to a wide range of ecological conditions (Oginosako et al., 2005; Essien et al., 2012; Tilney et al., 2018). Moreover, these species enhance soil fertility through nitrogen fixation (Wekesa, 2018) hence their close association. Tabernaemontana stapfiana, Allophyllus abyssinicus, Milicia excelsa, Cordia Africana and Vachellia (Acacia) xanthophloeae require moist and wet soil conditions (Omoro et al., 2010) which are commonly found in the crop farming system which is frequently flooded during the rainy season. These species also do well in adequately aerated soils typical of cultivated areas and enrich soil either through nitrogen fixation or organic matter addition through leaf litter fall. They are very valuable in improving soil fertility in crop farming areas (Wekesa, 2018).
Smit et al., 2006 and Mullah et al., 2013) found evidence showing that dominant tree species can either facilitate or inhibit recruitment of other forest species. Facilitation in which the presence of one plant species is beneficial to the growth and survival of another plant species in its proximity, often occur in stressful environments such as cold, saline and arid ecosystems. In the semi-arid livestock production zone, the dominant tree species which are stress-tolerant ameliorated adverse environmental conditions in their immediate environment through provision of shade and soil nutrients hence strongly influencing the occurrence of less dominant tree species. Dominant species such as V. nubica, G. bicolor and E. capensis which fix nitrogen, provided favourable conditions to facilitate growth of other species. Mullah et al., (2013) also found that nitrogen-fixing legumes like A. gummifera facilitate growth of other plants in naturally regenerating degraded abandoned fallows in the tropics. Restoration initiatives should therefore prioritize dominant tree species due to their critical role in facilitating the establishment of less dominant tree species.
g) Interaction between dominant and rare tree species along River Lumi riparian ecosystem
The CCA model was not significant for the interaction between dominant and rare tree species (Albizia glaberrima, Albizia gummifera, Bridelia micrantha, Xymalos monospora, Senna denimetria, Senna spectabilis, Croton macrostachyus, Rauvolfia caffra, Ehretia petiolaries, Taprafisc, and Sorindeia madagascariensis) along River Lumi riparian ecosystem . Vachellia (Acacia) nubica was found to co-exist with Xymalos monospora while Grewia bicolor co-existed with Albizia glaberrima, Senna denimetria and Croton macrostachyus. Ekerbergia capensis occurred in association with Rauvolfia Caffra and Albizia gummifera, while Trichiliaemetica was found to co-exist with Ehretiapetiolaries and Taprafisc. Tabernaemontana stapfiana grew together with Bridelia micrantha, Sorindeia madagascariensis and Senna spectabilis (Figure 8).
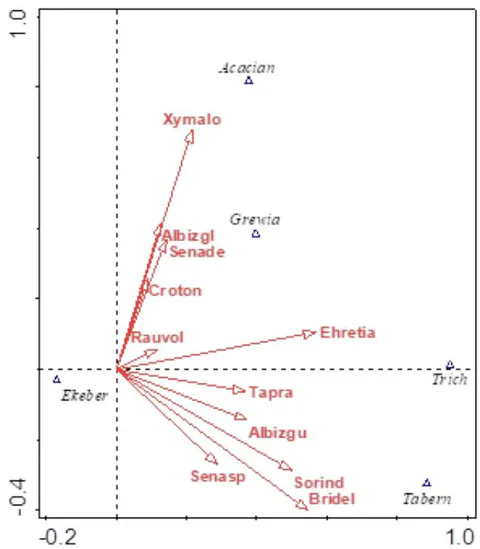
Vachellia (Acacia) nubica was associated with Xymalos monospora whereas Grewia bicolor grew together with Albizia glaberrima, Senna denimetria and Croton macrostachyus. Ekerbergia capensis occurred with Rauvolfia Caffra and Albizia gummifera, while Trichilia emetica occurred with Ehretia petiolaries and Tapra fisc. Tabernaemontana stapfiana occurred with Bridelia micrantha, Sorindeia madagascariensis and Senna spectabilis. A. nubica and X. monospora compete aggressively to form thickets (Pratt and Gwynne, 1977; Oginosako et al., 2005), and are associated with high levels of disturbance hence their occurrence together mainly in disturbed areas along River Lumi riparian ecosystem. The close association between Grewia bicolor, Albizia glaberrima, Senna denimetria and Croton macrostachyus species is due to their drought tolerance and are commonly found in dry areas with limited moisture supplies as confirmed by Mullah et al., (2013). These species are also early colonizers in forest regrowth and are characteristic of secondary forests
(Omoro et al., 2010). Ekerbergia capensis, Rauvolfia Caffra and Albizia gummifera are agro-forestry tree species hence their close association (Omoro et al., 2010). The roots of A. gummifera contain Bradyrhizobium bacteria that fix nitrogen in the soil (Wekesa, 2018), while capensis is a good soil stabilizer (Tilney et al., 2018). Both capensis and caffra experience heavy leaf fall which increases humus content of the soil especially during the dry season (Omoro et al., 2010; Mullah et al., 2013). Therefore, dominant and rare tree species with similar physiological characteristics occurred together. Similar to their effect on less dominant species, the dominant tree species ameliorated adverse environmental conditions thereby facilitating the growth of rare species which are often distributed in narrow areas with special microclimates (Chen et al., 2014). Rare tree species play an important role in biodiversity conservation (Mullah et al., 2013; Chen et al., 2014)), hence proper matching of dominant and rare tree species is critical for their growth and survival, and for successful restoration initiatives.
h) Livelihood sources and their contribution to household income
Mean household income (KES per annum) derived from mixed, crop and livestock production value chain along River Lumi riparian ecosystem was not significantly different . However, the crop farming enterprise yielded the highest income . This was followed by the mixed farming system and livestock production system . Similarly, the mean household income derived from business was not significantly different in the three land use systems , although households in crop farming system derived more income , than those in mixed farming system , and livestock production system . Mean household income derived from employment was also not significantly different in the three land use systems . Income derived from employment in livestock production system was, however, higher as compared to mixed farming system and crop farming system . A similar trend was observed in the mean household income derived from remittance which was not significantly different in the three land use systems even though the income was higher in crop farming system than in mixed farming system and livestock production system . Overall, the average household income was higher in the mixed farming system than in the crop farming and livestock production land use system (Figure 9).
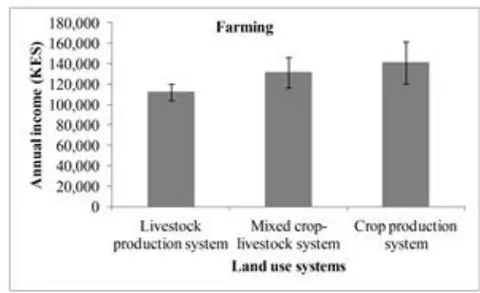
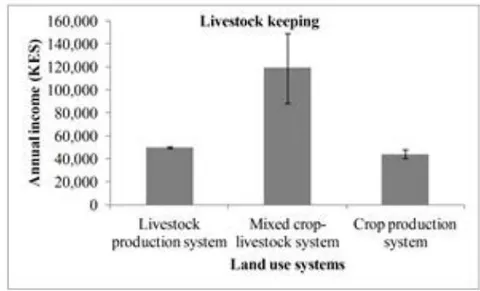
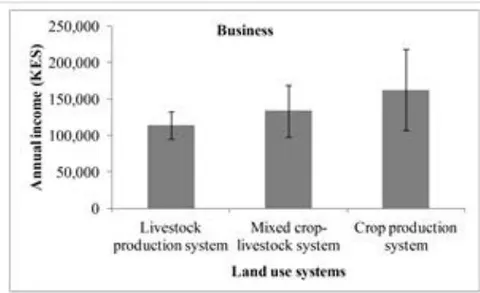
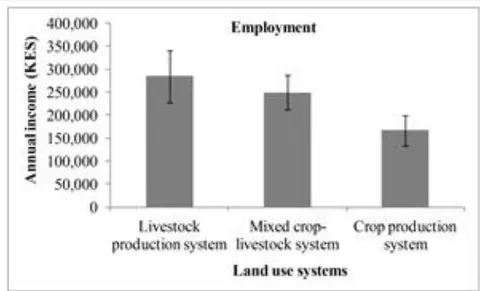
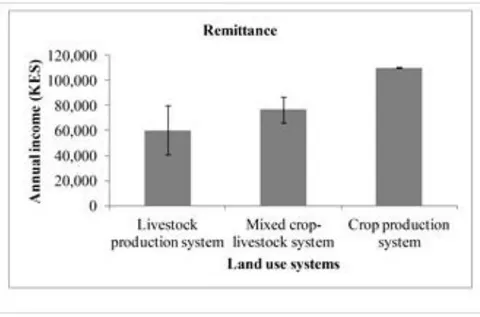
Crop farming and livestock production were undertaken for commercial and subsistence purposes. The main crops grown were maize, bananas, tomatoes, onions, leafy vegetables, green grams and beans, while the main livestock kept were cattle, goats and sheep. The area under crop production increased considerably in the seven-year period between 2011 and 2018 in response to the need to diversify crop farming to ward off the negative impacts of climate change. Increased human population and concomitant expansion of the coastal towns of Voi, Mombasa and Malindi triggered increased demand of agricultural products. The pressure for increased crop yields and agricultural intensification is a significant driver for increased agricultural mechanization in crop irrigation farming and utilization of industrial fertilizers and pesticides (Foley et al., 2005, Muli, 2014). Although there was a decline in livestock numbers in River Lumiriparian ecosystem over the same period there was an influx of livestock from neighbouring pastoral communities and adjacent private ranches. Ecological degradation attributed to defoliation impacts from increased livestock densities was witnessed in the riparian ecosystem. Similar effects have been echoed in the studies of Lambin and Geist, 2006 who found that increased demand for food was associated with increased agricultural production leading to declines in natural vegetation and grasslands.
In the current study, there was evidence of human induced transformation of riparian forest structure as well as shifts in botanical composition of dominant, less dominant and rare species as reported elsewhere in this study. This is a clear testimony of the diminishing ecosystem integrity and resilience of River Lumi riparian ecosystem. Studies by Dibaba et al., 2020 revolving around the impacts of agriculture driven land use and land use land cover change in Finchaa Catchment in North-Western Ethiopia revealed that decrease in crop yields and reduced agricultural profitability, loss of biodiversity and concomitant loss of habitat and soil fertility were associated with weakened livelihood support systems.
Shackleton et al. (2007) and Kalaba et al. (2010) have adduced evidence indicating that poor communities are most affected by the negative impacts of environmental degradation in view of the direct dependence of their livelihood support system on land and natural resources.
i) Influence of socio-economic factors on production systems
Evaluations of interactions of factors of production embracing land income and land tenure, education levels as well as demographic attributes of gender, household size indicated negative Spearman rank correlation between household size and gender distribution (r = -0.209; p = 0.000), household size and land tenure (r = -0.072; p = 0.169), household size and household response to degradation (r = -0.050; p = 0.355) and gender of household head and education level of household head (r = -0.166; p = 0.003). However, there was a positive relationship between household size and education level (r = 0.058; p = 0.273), Table 2.
| Variable | HH size | Gender HH | Education | Land tenure | HH Incom | Resp |
| HH size | 1.000 | |||||
| Gender HH | -0.209* | 1.000 | ||||
| Education | 0.058 | -0.166* | 1.000 | |||
| Land tenure | -0.072 | 0.022 | -0.004 | 1.000 | ||
| HH Income | 0.019 | -0.170* | -0.016 | 0.075 | 1.000 | |
| Response | -0.050 | 0.025 | -0.028 | -0.022 | 0.016 | 1.000 |
Evidence has shown that community participation in conservation projects is important as it enhances local participation and flow of benefits to local communities, lessens potential resistance or conflict, helps to reduce implementation costs, and increases the likelihood of project success (Aganyira et al., 2020; Mogomotsi et al., 2020). However, despite its importance, community participation in conservation projects remains elusive for most rural communities in developing countries, and debates on the criteria for local participation remain critical (Aganyira et al., 2020).
There is evidence from the current study that household head did not influence household size/beit, house hold size had an influence on education and income levels. The likelihood of a greater number of educated people was associated with large households. There was also evidence that a high proportion of members from such households were engaged in several income generating activities contributing to household wealth. Gender of household head had an influence on land tenure and household response to degradation. As is the case for patriarchal rural African communities, land ownership is a preserve for male members of the household. Female members have delegated land use and land access rights. More male headed households responded to degradation of River Lumi riparian ecosystem through involvement in conservation initiatives than the female headed households. Decisions regarding the main land uses and livelihood activities such as commercial crop farming and livestock production were made by men who were also the greatest beneficiaries of economic returns from these activities. As such, men were more motivated to respond to degradation to prevent adverse effects on their livelihoods. Omollo et al., (2018) found that access to productive assets and other resources in the rural African context are strongly influenced by gender and female-headed households are constrained by limited access to natural resources. Male-headed households often have more access to productive resources such as livestock, land and finances compared to female-headed households, and are therefore more likely to adopt sustainable land
management practices than their female counterparts (Wasonga, 2009).
Land ownership rights authenticated by the possession of title deeds facilitated accessibility to credit facilities for land development and other revenue generating activities. This explains the positive relationship between land tenure and household income. Previous studies have authenticated that lack of individual land tenure rights often led to absence of commitment and was responsible for poor choices of land management practices and land degradation (World Bank 2019). Other studies conducted in East Africa (Alden Wily, 2018; Muraoka et al., 2018; Schurmann et al., 2020) that examined the relationship between land rights and involvement in environmental conservation at household level confirmed that land rights influence the adoption of sustainable land use practices. According to Carter et al., (1994), community engagement in long-term resource conservation activities was positively correlated with the potential to derive benefits from related land uses during the term of the rights of use, with more long-term investments being frequently made in registered land.
There was a positive interaction between household income level and response to degradation. Household wealth was a function of response to land degradation mitigation initiatives. Households with higher income levels demonstrated greater commitment in the mitigation of adverse consequences of degradation such as charcoal production and illegal logging. Previous studies on the impacts of poverty on environmental degradation in Katonga Basin in Uganda (Niringiye et al., 2010) established that poverty was a major driver of deforestation. Additional evidence from the Bruntland Commission report authenticates that poverty is a major driver of environmental catastrophies (World Commission on Environment and Development, 1987). Schurmann et al. (2020) research work in Arabuko Sokoke forest established that household income had an effect on participation in conservation activities. High poverty levels amongst forest adjacent households in Arabuko Sokoke forest were responsible for over-extraction of fuelwood and building material leading to forest degradation. Mogomotsi et al., (2020) who evaluated the drivers of community involvement in wildlife conservation in Botswana adduced evidence that showed that household income and education levels had a positive correlation with community participation in conservation initiatives.
Evidence from the current study indicates that household size and education level had no influence on household response to degradation. Instead, household willingness, motivation and conservation awareness among members of the household were found to be major determinants of response to degradation. According to Htay (2020), conservation attitudes of local communities, level of conservation awareness and benefits accrued from the protected area influenced conservation support amongst local communities. Other studies (Infield and Namara, 2001; Tessema et al., 2010; Htun et al., 2012; Karanth and Nepal, 2012) have also indicated that people's willingness to participate in conservation programmes are strongly linked to their attitudes. People with positive attitudes are more likely to have conservation supportive inclinations whereas those with negative attitudes are likely to behave in less supportive manners (Ajzen, 1991; Nepal and Spiteri, 2011; Allendorf, 2022). The negative correlation between household education level and response to degradation observed in this study is also apparent in the research work of Kassie (2017), who established that households with lower levels of education generally had low willingness to engage in sustainable land management activities. Households with high levels of education are often engaged in activities with higher economic returns. In River Lumi riparian ecosystem, household members with high levels of education mostly migrated to urban areas in search for employment opportunities while agricultural production was mainly undertaken by unskilled workforce. This explains the negative correlation between household education levels and response to degradation.
Elucidated evidence from this study and that of other research workers lends credence to the premise that sustainability of conservation projects is dependent on the welfare of local communities, and must take into consideration community concerns and aspirations, as well as their specific needs in their design and implementation (Oldekop et al., 2016; Aganyira et al., 2020). Enhanced conservation awareness and community access to benefits are critical in ensuring conservation effectiveness.
V. CONCLUSIONS
Irrigated crop production system in River Lumi flood plain plays an important role in tree diversity conservation and has the potential for integration of other plant material restorative initiatives for enhanced livelihood and conservation gains.
Soil-plant species interactions along River Lumi riparian ecosystem could be used to guide the selection of suitable tree species genotypes for rehabilitation of areas of degraded riparian ecosystems and enhancement of livestock fodder production potential.
Crop -livestock production system is a major contributor to household wealth and a source of ecosystem goods and services with a latitude for sustainable development for improved livelihoods.
The key socio-economic determinants of household response to ecosystem degradation were gender and household income. Accordingly, biodiversity restoration initiatives require appropriate involvement of both gender as well as the provision of economic incentives to communities to mitigate the adverse impacts of poverty on riparian ecosystem degradation.
Research findings of the current study are pivotal in the development of interventions for appropriate restoration of ecological integrity of riparian biodiversity hotspots and realization of Sustainable development Goals (SDGs), 6 (ensuring availability and sustainable management of water and sanitation for all), SDG 13 (combating climate change and its impacts) and SDG 15, (promotion of sustainable use of land ecosystems including forests).