I. INTRODUCTION
Onion (Allium cepa L.) is one of the most widespread crops in the world and is consumed by almost all peoples on the planet, regardless of ethnic and cultural origin, constituting an important element of family labor occupation (BOITEUX; MELO, 2004). It is the third most economically important vegetable in the world, and especially in Brazil (AGRIANUAL, 2016).
According to the systematic survey of agricultural production, the states with the largest productions were Santa Catarina, Rio Grande do Sul, Paraná, Minas Gerais, São Paulo, Goiás, Bahia, and Pernambuco, with harvests ranging from 55,460 to 509,389 tons (IBGE, 2017).
Given the relevance of this crop, research on onions is essential, especially for plant breeding programs. The aim of these programs, is to produce high-quality commercial products; thus, breeders need a broad genetic base and good breeding strategies to promote favorable genetic improvements in the crop (SANTOS, 2011).
One way for plant breeders to verify the existence of genetic variability in a given population is through genetic parameter estimates (VENCOVSKY, 1978). These are theoretical quantities that describe the genetic structure of quantitative traits, providing important information on the magnitude of the additive variance and the variance due to dominance shifts (RAMALHO; SANTOS; PINTO, 2004).
One of the most important parameters is heritability, which expresses the reliability of the phenotypic value as an estimator of the genotypic value in such a way that the greater it is, the greater the genetic gain by selection (CRUZ, 2005). Another useful parameter for selection efficiency is the relationship between the coefficient of genetic and environmental variation, which evaluates the genetic proportion in relation to environmental variation (LIMA FILHO, 2015).
Besides the knowledge of genetic variability, it is necessary to know the genetic diversity and the existing correlations between the characteristics of interest. For selective breeding, studies involving genetic diversity among a group of genotypes are extremely relevant for the knowledge of the genetic resources available. This kind of research can employ multivariate techniques, especially cluster analysis, which allows combining multiple information of each genotype, facilitating selection from a combination of variables and identification of superior genotypes (CRUZ; REGAZZI; CARNEIRO, 2014).
Correlation analysis determines the degree of association between characters that can contribute to the adoption of indirect selection, especially among characters that present complications regarding selection due to low heritability or measurement and identification problems (TEIXEIRA et al. 2012; CRUZ; REGAZZI; CARNEIRO, 2012).
In view of the above, the objective of the present study is to evaluate genetic parameters and diversity, in addition to the phenotypic and genotypic correlations of characters related to onion production.
II. MATERIALS AND METHODS
The experiment was conducted in an agricultural experimental station in Uberlândia, Minas Gerais (MG), Brazil (18° 55' S latitude, 48° 16' W longitude, and 873 m altitude) in 2017. This study analyzed a set of genotypes consisting of 53 advanced strains. Some of the genotypes studied originated from O. P. populations (open pollination) adapted to cultivation in Brazil, especially those predominant in the south of the country, some from the onion breeding program maintained by the company in California, USA, and some from crosses between special subjects of these two origins (F2).
The strains were obtained through successive self-fertilizations (which varied from 4 to 5) and/or selffertilizations intercalated with intercrossing sibs between 2-3 plants. The criterion to define if the genotype would be successively self-fertilized or if it would advance through one or more generations in sib intercalated with self-fertilization or not, was based on the phenotypic state of seed production. Genotypes with lower seed production were subjected to sibs (2-3 plants) rather than being successively self-fertilized. In genotypes of advanced strains, an average of five generations of advancement through self-fertilization and/or sibs were involved.
A randomized block design (RBD) with two repetitions was used. Each plot consisted of a 1 m x 90 cm bed, with five rows spaced 20 cm apart, with plants spaced 5 cm apart, totaling to 100 plants per plot. For the characteristics that were not directly measured, scores from 1 to 9 were assigned, where 1 represented the worst value and 9 the best value of the variable. These characteristics were evaluated at plot level.
Sowing was performed in March and transplantation in May 2017. The beds were prepared and fertilized following the recommendations for onion crop. The morpho-agronomic characters evaluated were: plant vigor, a score (1-9) was assigned for plant vigor at 90 days after sowing (DAS) by assessing leaf diameter, plant height, and number of leaves; pseudostem 'neck' diameter: 1 for pseudostem with excessive thickening and 9 for those with less thickness; plant architecture: 1 for prostrate, 9 for erect; leaf waxiness: 1 for absence of wax and 9 for presence of a lot of wax; drying of leaf tips: the highest score was assigned to plants that did not present drying of leaf tissues and the lowest grade for the inverse situation; and plant cycle: quantity of days from sowing date to harvest.
The following evaluations were performed on the bulbs after their harvest: bulb mean mass, in grams; bulb density, d = mass/volume, g. cm-3; bulb color, with the highest score given for bulbs with dark brown color; bulb shape: with 1 for flat bulbs and 9 for rounded bulbs; uniformity of bulb shape: the greater the predominance of a shape in the plot, the higher the score; bulb firmness: with the aid of a penetrometer with a 6-mm tip, unit kgf.cm-2; durability after harvest of bulbs: the percentage of marketable bulbs was evaluated after 60 days of storage in ambient conditions.
All characters in the present study were treated as quantitative, considering the study by Sneath and Sokal (1973). Since the values of the multi-categorical characters could be ordered, i.e., they are of ordinal nature and reported on a scale, it is possible for them to be analyzed as quantitative variables.
Genetic variability among the genotypes was verified using analysis of variance and genetic parameters, such as broad-sense heritability and the relationship between genetic and environmental coefficients of variation, in addition to experimental coefficient of variation.
Genetic dissimilarity was estimated using the generalized Mahalanobis distance. Data were grouped using the hierarchical method, unweighted pair-group method using arithmetic averages (UPGMA), and an optimization method, Tocher.
A dendrogram was obtained from the UPGMA, which was defined by the genotypes with the highest similarity. The adequacy of the hierarchical grouping method was verified using the cophenetic correlation coefficient. The relative importance of each variable was estimated by the Singh's method (1981). The performance of each group, formed by the UPGMA, was evaluated based on the average of each group.
Phenotypic and genotypic correlations were evaluated. The significance of the phenotypic correlation was estimated using the t-test with n-2 degrees of freedom, where n is the number of genotypes evaluated. The significance of the genotypic correlations was evaluated by the bootstrap with 5,000 simulations.
Path analysis was used to estimate direct and indirect effects. In this analysis, the mean mass of bulbs was considered as the main dependent variable, and it was performed only when its correlations with other characters had correlation estimates and were significant. Prior to the analysis, the degree of multicollinearity was calculated following the criteria established by Montgomery and Peck (1981).
The Genes software (CRUZ, 2013) was used to perform the analyses, and the dendrogram was generated using the graphics and dendextend packages in the R version 3.5.2 software (R CORE TEAM, 2018).
III. RESULTS AND DISCUSSION
This study found the existence of genetic variability among the genotypes for most of the characters evaluated at the significance level of 1% by the F test (Table 1), showing that strain selection is possible. The variables that were not significant were neglected in the subsequent analyses.
| Characters | MS | (%) | CVg/CVe | CV (%) |
| Plant vigor | 1.66** | 56.99 | 0.81 | 14.26 |
| Pseud. diam. | 0.40* | 41.03 | 0.58 | 7.41 |
| Plant archit. | 1.54** | 49.80 | 0.70 | 15.80 |
| Leaf waxiness | 1.25** | 52.08 | 0.73 | 11.11 |
| Leaf dryness | 4.48** | 76.94 | 1.29 | 17.89 |
| Cycle | 415.57** | 93.74 | 2.73 | 2.99 |
| Mean mass | 96816.85** | 70.09 | 1.08 | 14.99 |
| Density | 0.00 | 0.00 | 7.94 | |
| Bulb color | 0.92** | 87.48 | 1.86 | 5.09 |
| Bulb shape | 0.63** | 71.46 | 1.11 | 6.06 |
| Shape unif. | 0.71** | 71.24 | 1.11 | 6.31 |
| Bulb firm. | 3.22** | 88.40 | 1.95 | 9.43 |
| Post-harvest | 41.06** | 82.98 | 1.56 | 28.47 |
The heritability ( ) of most characters showed moderate to high values ( ). The vigor of plants did not show the highest values of heritability (56.99%) in this study. The mean mass variable is indicative of crop production, and the heritability of this variable, with a value of 70.09%, was considered moderate according to the literature.
The results for heritability can be explained by the additive effect present in the advanced genotypes, resulting from their genetic homozygosity. As for the bulb density variable, several genes might be responsible for it, which would explain its low heritability value and the small density values. The genetic gain from selection for this variable seems to be very low.
Porta et al. (2014) studied the heritability of characters in onion landrace and S1 varieties and obtained the highest value of broad-sense heritability for the characteristics of dry matter, maximum leaf length and soluble solid content, respectively. Some authors attribute relative importance to the characteristics, dry matter and soluble solids content, due to their direct relationship with post-harvest, because they imply the storage capacity and commercial quality of bulbs. This study considered the storage period, and the heritability was high (82.98%).
Heritability allows predicting genetic gains in the future selection cycles. Traits with higher heritability will bring greater gains. Thus, the characters' cycle, mean mass, color, shape, and uniformity of bulb shape, in addition to firmness and preservation after harvest, tend to respond favorably to the selection process for genetic gains. Oliveira (2015) estimated the broad-sense heritability of total and commercial bulb yields of Valenciana onion populations in two environments, and the highest values obtained were 77% and 81%, respectively.
Similarly, the inferences about the success of the selection can be made by analyzing the values of the CVg/CVe ratios. Table 1 shows values above one unit for leaf dryness, cycle, bulb color, bulb shape, bulb shape uniformity, mean mass of bulbs, bulb firmness, and post-harvest durability. The characteristic that presented the highest CVg/CVe ratio was cycle, and the lowest was bulb density, which also presented low heritability.
The study of the relationship between the coefficients of genetic and environmental variation (CVg/CVe) indicates the possibility of gain with selection. This ratio serves as a parameter of the superiority of the genetic components in comparison to the environmental components. When this ratio is , the possibility of obtaining gains by selection is high (TORRES, 2015).
In this study, with the lowest CV values for the characteristics: cycle, color, shape, and uniformity of bulb shape, the experimental coefficients of variation were corroborated by those observed in the literature, reinforcing the accuracy of the statistical inferences made for these characteristics. The experimental CV of the advanced strains varied from 2.99% (cycle) to 28.47% (post-harvest durability).
CV is a measure of dispersion for estimating the experimental precision. The lower the CV, the greater the experimental accuracy, although the idea of accuracy is inherently related to each research area (RODRIGUES, 2013); therefore, for most of the characters evaluated, the experimental precision was medium to high.
Some studies by other authors showed that the CV values obtained in this study are in the range that is commonly obtained in research with onions. Ricci et al. (2014) reached values of 12.5%, 12.5%, and 13.7%.
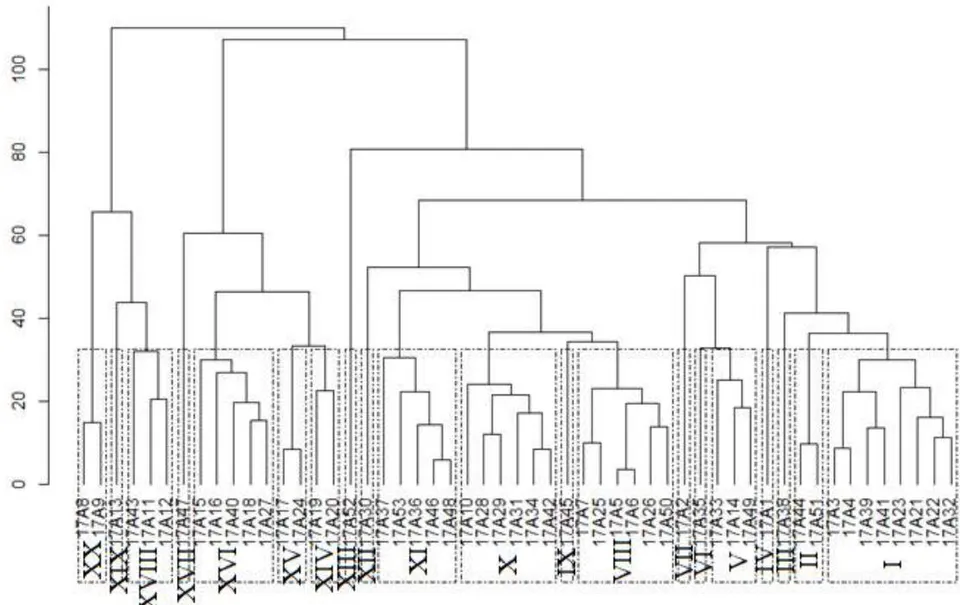
In the UPGMA, the delimitation of groups obtained in dendrograms can be determined through a visual examination and subjectively observing the points of high-level change in the dendrogram (CRUZ; REGAZZI; CARNEIRO, 2012). Following this assumption, Figure 1 shows the formation of 20 groups with 32.5% dissimilarity as the delimitation criterion.
The cophenetic correlation coefficient (CCC) obtained, r = 0.64 (at 1% probability, i.e., ), being significant for clustering, allowed visual inferences through the dendrogram.
Some studies by Filho and Guadagnin (2011) showed that in experiments with many cultivars and variables, there is a tendency for lower CCC; thus, corroborating the CCC value obtained in this study.
Of the 20 groups formed, groups I, VIII, X, XI, and XVI together were responsible for grouping 47.2% of the genotypes studied. Moreover, a considerable number of groups contained only one genotype each. These were groups III, IV, VI, VII, IX, XII, XIII, XVII, and XIX. In other words, their isolation in one group shows that they present an accentuated degree of divergence compared to the others.
The Tocher optimization method, based on the Mahalanobis matrix, segregated the 53 genotypes into 19 groups (Table 2), of which 56.6% of the genotypes were gathered in groups I, II, and III, and the rest in smaller groups.
The UPGMA and Tocher methods gave similar results for the number of groups formed. In both the methods, genotypes 17A1, 17A2, 17A13, 17A30, 17A38, 17A47, and 17A52 formed one group each, showing once again that they differed considerably from the rest of the genotypes studied. Moreover, the UPGMA method presented nine groups with only one genotype, while the Tocher method formed 12 groups.
In both the methods, group V was practically identical - UPGMA: 17A33, 17A14, and 17A49, and Tocher: 17A33, 17A14, 17A49 and 17A35. So were the groups XVIII and VI with genotypes 17A12 and 17A43, and groups XX and IV with genotypes 17A8 and 17A9 in UPGMA and Tocher, respectively. In the other groups, there was not much similarity.
| Groups | Genotypes |
| I | 17A5 17A6 17A26 17A34 17A25 17A7 17A50 17A42 17A29 17A31 17A28 17A48 17A36 17A46 |
| II | 17A17 17A24 17A18 17A16 17A19 17A40 17A27 |
| III | 17A3 17A4 17A22 17A41 17A39 17A21 17A32 17A44 17A51 |
| IV | 17A8 17A9 |
| V | 17A14 17A49 17A33 17A35 |
| VI | 17A11 17A12 17A43 |
| VII | 17A23 17A53 |
| VIII | 17A15 |
| IX | 17A30 |
| X | 17A20 |
| XI | 17A10 |
| XII | 17A37 |
| XIII | 17A1 |
| XIV | 17A38 |
| XV | 17A52 |
| XVI | 17A2 |
| XVII | 17A13 |
| XVIII | 17A45 |
| XIX | 17A47 |
From the mean of the 12 variables in the groups generated by the UPGMA method, it is evident that groups XIV, XVIII, and XIX stood out with highest values in the greatest number of characters of interest for onion production (Table 3).
| Groups | VIG | PD | ARQ | LW | LD | PC | MBM | BC | BS | UNI | FIR | POS |
| I | 6 | 7 | 6 | 7 | 5 | 170 | 110.3 | 6 | 7 | 7 | 5.7 | 11 |
| II | 8 | 6 | 6 | 8 | 5 | 182 | 115.0 | 6 | 7 | 7 | 5.2 | 8 |
| III | 7 | 7 | 5 | 8 | 4 | 165 | 113.3 | 5 | 7 | 6 | 5.5 | 14 |
| IV | 6 | 7 | 8 | 7 | 3 | 181 | 140.0 | 7 | 6 | 8 | 4.8 | 4 |
| V | 6 | 6 | 5 | 7 | 5 | 156 | 136.8 | 7 | 7 | 7 | 6.5 | 11 |
| VI | 6 | 7 | 5 | 7 | 6 | 174 | 151.0 | 7 | 7 | 6 | 5.6 | 11 |
| VII | 6 | 7 | 4 | 6 | 7 | 170 | 133.3 | 6 | 6 | 8 | 6.3 | 13 |
| VIII | 5 | 7 | 5 | 7 | 7 | 184 | 104.6 | 7 | 7 | 7 | 6.3 | 3 |
| IX | 6 | 7 | 4 | 7 | 6 | 182 | 85.5 | 7 | 7 | 6 | 5.7 | 2 |
| X | 5 | 7 | 6 | 7 | 5 | 185 | 79.7 | 7 | 7 | 7 | 6.7 | 5 |
| XI | 6 | 7 | 6 | 8 | 7 | 184 | 114.1 | 7 | 7 | 7 | 7.6 | 9 |
| XII | 7 | 5 | 6 | 7 | 8 | 182 | 115.3 | 7 | 8 | 8 | 6.3 | 6 |
| XIII | 7 | 6 | 7 | 7 | 5 | 189 | 95.0 | 6 | 8 | 8 | 7.5 | 3 |
| XIV | 5 | 7 | 6 | 7 | 8 | 167 | 106.1 | 7 | 8 | 8 | 5.5 | 13 |
| XV | 5 | 6 | 5 | 8 | 7 | 151 | 145.0 | 7 | 8 | 8 | 6.2 | 15 |
| XVI | 7 | 6 | 6 | 7 | 6 | 149 | 119.2 | 7 | 8 | 7 | 5.8 | 14 |
| XVII | 8 | 6 | 6 | 8 | 8 | 145 | 169.0 | 6 | 8 | 8 | 4.6 | 14 |
| XVIII | 7 | 7 | 5 | 7 | 5 | 153 | 114.9 | 8 | 7 | 7 | 8.5 | 13 |
| XIX | 7 | 7 | 6 | 8 | 6 | 148 | 122.8 | 7 | 7 | 6 | 10.8 | 15 |
| XX | 5 | 7 | 6 | 6 | 4 | 166 | 119.8 | 8 | 6 | 8 | 8.9 | 15 |
Table 3 shows that groups V, XV, XVI, XVII, and XX presented the most precocious genotypes (with shorter plant cycles), and stood out for bulb-related characters (color, shape, plot uniformity, mean mass, and post-harvest).
These results point out that the combination between the superior and contrasting genotypes for onion production of groups V, XIV, XVIV, XVI, XVII, XVIII, XIX, and XX, will enable the expansion of favorable genetic variability.
The characters plant cycle, bulb firmness, and bulb color together comprised more than 50% of the relative contribution to the divergence of the genotypes. The remaining characters showed smaller relative contribution and therefore were less influential for the divergence (Table 4).
Six significant phenotypic correlations were found using the t-test. The estimates ranged from 0.28 to 0.77, showing a low to moderate degree of association (Table 5). Most of the genotypic correlations were higher than the phenotypic ones, and presented the same sign, positive or negative.
The phenotypic association was probably minimized by the environment. The degree of freedom improves the estimates as a result of the increased number of repetitions. In addition, it improves the estimates of genotypic variances, and consequently, the estimates of correlations.
| Characters | S.j. | Value (%) |
| Cycle | 28196.41 | 25.35 |
| Bulb firmness | 15665.36 | 14.08 |
| Bulb color | 12028.74 | 10.81 |
| Bulb weight | 8592.56 | 7.72 |
| Bulb post-harvest durability | 8530.50 | 7.67 |
| Plot uniformity of bulbs | 8168.16 | 7.34 |
| Bulb shape | 7657.19 | 6.88 |
| Leaf dryness | 7062.31 | 6.35 |
| Architecture | 4494.53 | 4.04 |
| Vigor | 4113.94 | 3.69 |
| Leaf waxiness | 3890.72 | 3.49 |
| Pseudostem diameter | 2789.14 | 2.50 |
Characters S.j. Value (%) Cycle 28196.41 25.35 Bulb firmness 15665.36 14.08 Bulb color 12028.74 10.81 Bulb weight 8592.56 7.72 Bulb post-harvest durability 8530.50 7.67 Plot uniformity of bulbs 8168.16
| PD | ARQ | LW | LD | PC | MBM | BC | BS | UNI | FIR | POS | ||
| VIG | rp | -0.42** | 0.19 | 0.23 | -0.14 | -0.22 | 0.28* | -0.21 | 0.18 | -0.13 | -0.06 | 0.16 |
| rg | -0.41 | 0.20 | 0.33 | -0.22 | -0.23 | 0.25 | -0.36 | 0.39 | -0.33 | -0.14 | 0.22 | |
| PD | rp | 0.09 | -0.02 | 0.00 | 0.14 | -0.33* | 0.27 | -0.24 | -0.15 | 0.23 | -0.12 | |
| rg | 0.18 | -0.04 | 0.02 | 0.16 | -0.53+ | 0.46 | -0.62 | -0.31 | 0.44+ | -0.17 | ||
| ARQ | rp | 0.13 | 0.00 | -0.05 | 0.00 | 0.00 | 0.26 | 0.27 | -0.11 | 0.02 | ||
| rg | 0.32 | 0.02 | -0.10 | -0.17 | 0.07 | 0.62 | 0.51 | -0.12 | 0.09 | |||
| LW | rp | 0.27 | -0.14 | 0.18 | 0.07 | 0.23 | -0.14 | -0.13 | 0.02 | |||
| rg | 0.48 | -0.21 | 0.23 | 0.12 | 0.49 | -0.44 | -0.11 | 0.09 | ||||
| LD | rp | 0.02 | 0.12 | 0.09 | 0.13 | -0.01 | 0.00 | -0.03 | ||||
| rg | 0.00 | 0.20 | 0.12 | 0.19 | 0.02 | -0.01 | -0.04 | |||||
| PC | rp | -0.50** | 0.10 | -0.28 | -0.01 | -0.05 | -0.77** | |||||
| rg | -0.64++ | 0.13 | -0.35 | -0.01 | -0.04 | -0.85++ | ||||||
| MBM | rp | -0.21 | 0.19 | 0.10 | -0.03 | 0.49** | ||||||
| rg | -0.22 | 0.31 | 0.08 | -0.11 | 0.70++ | |||||||
| BC | rp | -0.19 | 0.00 | 0.54 | -0.20 | |||||||
| rg | -0.26 | -0.03 | 0.59 | -0.21 | ||||||||
| BS | rp | 0.02 | -0.18 | 0.30 | ||||||||
| rg | 0.12 | -0.22 | 0.39 | |||||||||
| UNI | rp | -0.10 | 0.05 | |||||||||
| rg | -0.16 | 0.13 | ||||||||||
| FIR | rp | 0.15 | ||||||||||
| rg | 0.20 |
Phenotypic correlations have genetic and environmental causes; however, only the genetic ones are heritable, implying their use in guiding selective breeding programs (CRUZ; REGAZZZI; CARNEIRO, 2012). Therefore, the genetic phenotypic correlation has to receive special attention.
A negative and significant genetic correlation between pseudostem diameter and mean bulb mass (0.53), plant maturity cycle and mean bulb mass (-0.64), and plant maturity cycle and bulb post-harvest durability (-0.85) was identified, showing that one characteristic increases at the expense of another.
The correlations between mean bulb mass and post-harvest were significant with an emphasis on the genetic correlation (rp = 0.49** and rg = 0.70++). This result shows a direct relationship between these characteristics, and a possibility of performing indirect selection. In a study on soybeans, Machado et al. (2017a) confirmed that indirect selection by the number of pods per plant is efficient to select more productive plants.
The correlation between plant maturation cycle and mean bulb mass possibly reflects the interference of photoperiod that was probably insufficient for plant maturation and bulb formation (cycle), which favors lower mean mass. According to Singh et al. (2019), photoperiod plays a key role in the development of different phenophases.
If the photoperiod requirement for bulb formation is between 12 to 14 hours for Brazilian conditions (WAMSER et al., 2012), a better formation and a larger bulb size would be expected in a given period of time (cycle). It is evident, therefore, that the grouping of germplasms with similarity in photoperiodic requirements is necessary for studies involving characteristics related to production, such as pseudostem diameter, cycle, and mean bulb mass. In this experiment, however, a large number of genotypes with variations in photoperiodic requirements were evaluated, which may explain these results.
Aditika, Priyanka and Sharma (2015) studied 21 onion genotypes, and observed associations among characters related to onion bulb yield. Similarly, in this study, the authors have found significant genetic associations between bulb weight and neck thickness, and between bulb weight and number of days to taken to reach plant maturity. However, conversely, the correlations found by the authors were positive. These results confirm how the heterogeneity of the genotypes studied and the climatic conditions can affect the characters in question.
The estimated correlation between the variables plant maturation cycle and post-harvest bulb harvest showed high magnitude, but in negative association, indicating that plants that attain maturity early have a better post-harvest preservation. However, part of the effect of the high negative correlation between these two characters may also have come from the fact that some genotypes have poor bulb formation, due to the short photoperiod, which contributes greatly to lower post-harvest preservation.
From the correlations between mean bulb mass and post-harvest, it is assumed that heavier the bulb, greater is its preservation post-harvest. On the other hand, lighter bulbs tend to have lower post-harvest preservation. It is worth considering that the same effects explained for previous correlations, where bulbs of small size, due to malformation by photoperiodic insufficiency, also tend to have a lower post-harvest preservation.
The study of correlations has great relevance when it comes to quantifying the magnitude and direction of factors in determining characters, however, the direct and indirect effects of these factors are not given due importance. On the other hand, path analysis allows the unfolding of correlations of direct and indirect effects of the characteristics on a variable (CRUZ; REGAZZI; CARNEIRO, 2012).
In this study, the opposite association observed between the diameter of the pseudostem and the mean bulb mass was possibly due to the fact that in this correlation the mean mass of bulbs is greatly influenced by the photoperiod required for their formation, as when the photoperiod is insufficient, which probably occurred in this experiment, the pseudostem is thicker. It also shows that it is not feasible to use these characters for indirect selection.
The mean bulb mass showed significant genetic correlations > 0.5 with more than one variable (diameter of the pseudostem, cycle of maturation of the plants, and post-harvest preservation of bulbs); thus, a path analysis was performed to check if they really have strong cause-and-effect relationship.
The variables studied in the path analysis did not present multicollinearity problems. The low value of the coefficient of determination of the path (0.35) and the high effect of the residual variable (0.80) shows that the cause-and-effect relationship between the variables studied are weak (Table 6).
The estimation of direct genotypic effects showed that post-harvest preservation of bulbs had the greatest direct effect on the mean bulb mass. The positive indirect effect of the maturation cycle of the plants influenced the positive correlation with the mean mass of bulbs, and the diameter of the pseudostem was also influenced in the same way but to a lesser degree.
| Characters | Phenotypic effects | Genotypic effects |
| Direct effect PD/MBM | -0.267 | -0.430 |
| Indirect effect via PC | -0.040 | -0.031 |
| Indirect effect via POS | -0.029 | -0.078 |
| Total | -0.338 | -0.539 |
| Direct effect PC/MBM | -0.276 | -0.195 |
| Indirect effect via PD | -0.039 | -0.068 |
| Indirect effect via POS | -0.189 | -0.381 |
| Total | -0.505 | -0.645 |
| Direct effect POS/MBM | 0.245 | 0.449 |
| Indirect effect via PD | 0.032 | 0.075 |
| Indirect effect via PC | 0.213 | 0.165 |
| Total | 0.492 | 0.690 |
| Coefficient of determination | 0.35 | 0.67 |
| Residual effect | 0.80 | 0.58 |
The direct effects showed the same sign as the correlations, but their magnitudes were low (less than the estimated residual effect), both for phenotypic and genotypic effects, proving that the explanatory variables (pseudostem diameter, plant cycle, and post-harvest bulbs) are not the main ones responsible for the variation of the main variable (mean bulb mass), and consequently, indirect selection is likely to have low efficiency.
The phenotypic and genotypic variations that were not explained by the path analysis were 80% and 58%, respectively. This predicts that only 20% and 42% of the variations in mean bulb mass at the phenotypic and genotypic level, respectively, were determined by means of the path analysis.
In this study, plant health was not considered in the evaluation because during the management of the crop, an efficient phytosanitary control was performed. However, Machado et al. (2017b) studied onion populations and observed a high correlation between plant architecture and Botrytis spp. Torres et al. (2016), in their experiments on Urochloa brizantha, also confirmed in their results that phenotypic expression reduced under the influence of the environment; therefore, this is a variable to be considered in future studies. Parvez et al. (2020) studied the performance of purple onions, and detected cultivars tolerant to purple spot disease, so they can be used as source material in selective breeding programs.
IV. CONCLUSION
The genetic parameters studied shows the possibility of gains in the selection for most of the characters evaluated. The study identified a wide genetic variability for the morpho-agronomic traits evaluated, allowing the discrimination of groups of divergent genitors in onion. The phenotypic and genotypic correlations showed low associations between the evaluated characters, making the use of indirect selection unfeasible.
ACKNOWLEDGMENTS
The authors thank the Federal University of Ceará (UFC) and BAYER Vegetable Seeds for the support in the conduction of the experiment, the Coordination for the Improvement of Higher Education Personnel (CAPES), the National Council for Scientific and Technological Development (CNPq), and the Minas Gerais State Agency for Research and Development (FAPEMIG) for supporting this study.