I. INTRODUCTION
The Loess plateau of China is an erosionprone region that is susceptible to the forces of wind and water, and has been called the "the most highly erodible soil on Earth" (Tian and Huang, 2000). The area covers hawhich includes ha of grassland, with 91.2% of that area being occupied by natural grassland. Grassland is the mot common terrestrial ecosystem on Earth with a crucial function of regulating climate and maintaining a balanced ecosystem (Belsky, 1992). Widespread stress practice, intensive cultivation, overgrazing and large-scale monocultures have caused the Loess plateau to acquiesce to soil erosion and a series of related ecoenvironment problems (Montalvo et al., 1997; Fu, et al., 2000; An et al., 2009). Environmental restoration, which aims to restore disturbed ecosystems, has been an important tool for mitigating human pressure on natural environments (Holl, et al., 2003) and for improving ecological services (Doren, et al., 2009). The Grain to Green program, a national ecological restoration program implemented in 1999, has made remarkable advances in vegetation recovery on the Loess plateau (Feng, et al., 2013). Vegetation restoration is the most effective method for abating soil erosion and degradation (Hou, et al., 2002; Montalvo, et al., 1997). Several countermeasures have been implemented including eco-environment rehabilitation using engineering and biological approaches (Wang, 2002). Natural grassland protection and restoration is one of the important parts of a vegetation restoration program (Kerri, et al., 2002).
Soil structure, especially the spatial distribution of OM within the organic-mineral matrix of soil, exhibits control over microbial mediated decomposition processes in terrestrial ecosystems (Oades, 1988; Van Veen and Kuikman, 1990; Golchin, 1994; Ladd, et al., 1996). It exerts a significant amount of influence over other edaphic conditions and the surrounding environment, and often imbibes a degree of stability to aggregates (Bronick and Lal, 2005). Soil aggregates are structural units, where a group of primary soil particles cohere to each other more strongly than to other surrounding particles (Andraski and Scanlon, 2002). Research indicates that soil aggregates greatly impact the soil microbial biomass and mineral nutrients reserves (Hernández-Hernández and López-Hernández, 2002; Villar, et al., 2004). Thus, the soil microbial biomass demonstrates a similarly positive relationship with soil structure, and microbial biomass shows significantly positive relationships with aggregate size and stability (Gupta & Germida, 1988; Drury, et al., 1991; Jocteur-Monrozier, et al., 1991; Ghoshal and Singh, 1995). When assessing the effects of disturbances on soil quality, Anderson and Domsch (1985) proposed the ratio of soil basal respiration to microbial biomass (microbial metabolic quotient, specific respiration of the biomass or , conceptually based on Odum's theory of ecosystem succession, is increasingly being used as an index of ecosystem development (Odum, 1969 and 1985; Wardle & Ghani, 1995). Soil respiration is a major determinant of the carbon balance, Hunt, et al. (2004) and Wohlfahrt, et al. (2005) show that the proportionally largest emission of comes from grassland soil. Furthermore, soil microbial biomass basal respiration and microbial metabolic quotient all respond readily to disturbance effects and provide an effective early waning for the deterioration of soil quality (Powlson, et al., 1987; Wardle, 1992; Wardle & Ghani, 1995). They have been used as indicators of change in soil organic matter that occur in response to land use alteration, tillage practices and soil pollution (Sparling et al., 2003; An et al., 2009).
We hypothesize that the years under grassland restoration effects soil structure formation which consequently effects the distribution of soil microbial biomass and microbial metabolic quotient. The objectives of this study are (1) to investigate the distribution of soil microbial biomass and microbial metabolic quotient in different soil aggregate hierarchies at different restoration periods; (2) to determine the correlation between basic soil characteristics, and soil microbiological parameters; and (3) in this context, to examine soil aggregate stability.
II. MATERIALS AND METHODS
a) Study site description
The study area was located in Chinese Loess Plateau, the south of Ningxia Province (106° 25'-106° 30'E, 35° 59'-36° 20'N). The region has a sub-arid climate characterized by seasonal rainfall with periodic local flooding and drought; the average annual temperature was 6°C, and the average annual rainfall was 400-450 mm. The rainy season lasted from July to September and the rainfall in July accounting for 24% of the annual rainfall. Most of the land is at altitude of 1800-2040 m and is closely dissected by steep galleys (An et al., 2009). Grassland soils from three restoration years (30 years, natural grassland; 10 years, natural grassland; 1 year, abandoned grassland), were processed at the Yunwu Observatory for Vegetation Protection and Eco-environment.
b) Soil sampling collection
| Succesional Years | Dominant Species | Accompanying species | Elevation (m) | Slope gradient (°) |
| 30 | Thymus mongolicusStipa bungana | Stipa grandissArtemisia sacrorum.Artamisia scoparia | 1930 | 12 |
| 10 | Leymus secalinusThymus mongolicus | Artemisia scopariaPotentilla bifurcaStipa bungana | 1908 | 11 |
| 1 | Artemisia scopariaPotentilla bifurca | Thymus mongolicusHeteropappus altaicusThymus mongolicusStipa bungana | 1940 | 10 |
Samples were collected from 9 sites during May 2016 in each of the three restoration sites. For each restoration site (characterized by year), three samples/location were collected as replicates. An area of 50 m×50 m was selected for each of the 9 sites; within this area, three 10 m×10 m plots were selected and S-type multiple sampling methods were used for soil collection (0-20 cm). Soil sample collections were repeated 5 times in the field, mixed, transported to the laboratory and sieved (>5、5-3、3-2、2-1, 1-0.25 and <0.25 mm). Care was taken during sample preparation to minimize moisture loss and samples were divided in two. One section was preserve in 4°C for soil microbial measurements. The other was air dried for basic soil characteristics analysis. The water-holding capacity was determined by saturating each 100 cm3 turf sample with water and allowing it to drain at field capacity under cover for 48 h at ambient temperature; Duplicate soil
c) Sampling analysis
The soil samples were air dried and passed through a 2 mm sieve. The basic soil characteristics were analyzed through soil chemical and physical analyses (ISSCAS, 1981). Soil organic carbon was measured by wet digestion in a mixture of 5 ml of 0.136 mol/L potassium dichromate and 5 ml of concentrated sulfuric acid. Soil total nitrogen was measured using Kjeldahl digestion. Alkali-ExTR-N was measured using a micro-diffusion method in which was released from the soil sample by NaOH and then absorbed by boric acid. The ammonium borate product was titrated with 0.01 M HCl. Available phosphorus (Av-P) was extracted and measured in a buffered alkaline solution containing 0.5 M sodium bicarbonate. The extracts were quantified calorimetrically at 660 nm with a spectrophotometer (UV2300, Hitachi, Tokyo, Japan) (Xue et al., 2014). The readily available potassium was extracted from the soil with 1 mol/L and was measured using flame photometry. The soil pH was measured in water (1/2.5 w/v), and the moisture content was assessed by drying the samples in an oven at 105°C overnight.
Soil basal respiration was estimated through evolution at 25 °C in samples incubated for 10 days (Jenkinson and Powlson, 1976a). Measurements were made in the laboratory at 50% of field water holding capacity (WHC). respired was trapped in NaOH, and the residual NaOH was titrated with HCl(An et al., 2009).
The soil microbial biomass C, N and P levels were determined using the fumigation-extraction method. A 15 g sample of oven-dried, field-moist-equivalent soil (<2 mm) was fumigated with chloroform for 24 h with the chloroform being removed by repeated evacuation. The soil was reinoculated with a small amount of unfumigated soil and incubated at a constant temperature (usually 22 or 25) for 10 days at field capacity or at 50% of its water-holding capacity (approximately -0.01 MPa). An additional, unfumigated soil sample was used as a control (Jenkinson, 1976; Jenkinson and Powlson, 1976b; Xue et al., 2014). The soil microbial biomass carbon level was determined immediately using a TOC analyzer or the sample was preserved at -18 (Phoenix 8000, Tekmar Dohrmann, Mason, OH, U.S.A.). A value of 0.4 was chosen to calculate the total soil microbial biomass C (Wu et al., 1990). To determine soil microbial biomass N, fumigated and unfumigated samples were extracted via potassium persulfate oxidation and then measured using ultraviolet spectroscopy. The extract liquor was digested with alkaline auto-oxidation using 0.15 mol/L NaOH and 30 g/L with a 1:1 v/v mixture of oxidant and soil at 120-124 for 30 min (Zhou and Li, 1998; Xue et al., 2014). The concentration of N was determined colorimetrically using a spectrophotometer (UV2300, Hitachi, Tokyo, Japan) at 220 and 275 nm. A value of 0.54 was chosen to calculate the total soil microbial biomass N (Vance et al., 1987). The soil microbial P level was determined calorimetrically with a spectrophotometer. 2.5 g of fumigated and unfumigated soil was placed into a 150-ml flask containing 50 ml of 0.5 mol/L solution and 2 g of P-free active charcoal. 5 ml of Mo-Sb spectrochrometry solution was added for color development. After 30 minutes, the color was determined with a spectrophotometer (UV2300, Hitachi, Tokyo, Japan) at 700 nm. The microbial P was calculated using a factor of 0.40 (Hedley and Stewart, 1982; An et al., 2012).
III. RESULTS
a) Basic soil characteristics
| Soil Characteristics | Succesional years | ||
| 30 years | 10 years | 1year | |
| BD | 0.91 | 1.13 | 1.28 |
| MFC | 37.08 | 31.83 | 27.34 |
| Por. | 54.85 | 54.80 | 50.36 |
| SOC | 27.85 | 18.15 | 9.50 |
| TN | 3.10 | 1.88 | 1.17 |
| Ap-P | 3.56 | 3.37 | 2.71 |
| Ap-K | 166.24 | 241.69 | 153.04 |
| 14.08 | 4.21 | 4.53 | |
| 16.62 | 6.40 | 15.06 | |
| C: N | 8.87 | 8.26 | 8.26 |
| Inv. | 20.40 | 14.77 | 7.83 |
| Alk.-P | 12.43 | 9.99 | 5.95 |
| Ure. | 2.62 | 4.13 | 3.64 |
| 1065.49 | 683.72 | 358.96 | |
| 25.78 | 41.41 | 17.23 | |
| 19.99 | 15.74 | 2.56 | |
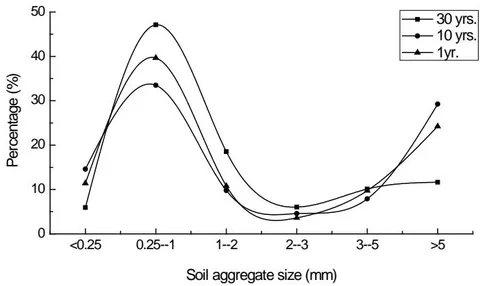
General soil characteristics for the various restoration years are shown in Table 2. As grassland recovery years increased, maximum field capacity (MFC), porosity (Por.), soil organic carbon (SOC), total nitrogen (TN), rapid available phosphorus (Ap-P), invertase (Inv), Alkal-phosphatase (Alk.-P), soil microbial biomass carbon ( ) and phosphorus ( ) also increased. However, restoration years also resulted in a decrease in bulk density (BD). The highest concentrations of soil microbial biomass nitrogen ( ), urease (Ure) and rapid available potassium (Ap-K) were found in 10 year grassland. The distribution of aggregate size class percentage varied among the grassland restoration sites (Fig. 1). The percentage of < 0.25 and > 5 mm aggregate sizes in 30 year natural grassland was lower than in 10 year. Lastly, soil aggregate composition in 30 year grassland was mainly concentrated between 0.25 and 5 mm.
b) Distribution of SOC and TN in various aggregate sizes
The concentration of SOC and TN associated with soil grain size increased with the number of years of grassland succession (Fig. 2 (a) and (c)). For 10- and 30-year natural grassland, the percentage of SOC in 1-2, 2-3 and 3-5 mm was higher than for other aggregate sizes. In 1 year abandoned grassland, the macro-aggregate size (>5 mm) showed the greatest SOC with rapid enhancement between 3-5 and 5 mm (Fig. 2 (b)). The trend in distribution of TN among the various aggregate classes in 10- and 30-year natural grassland was similar (i.e., stable between 15.79 - 17.64). However, significant changes occurred in 1year-abandoned grassland (Fig. 2 (d)). The percentage of TN (11.26) was lowest for micro-aggregates (<0.25 mm), highest in 0.25-1 mm (19.22), and remained at a lower yet steady level for 10- and 30-year (17.02-18.51).
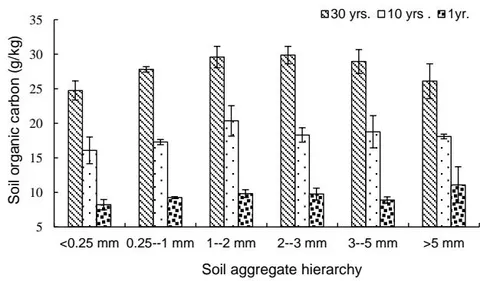
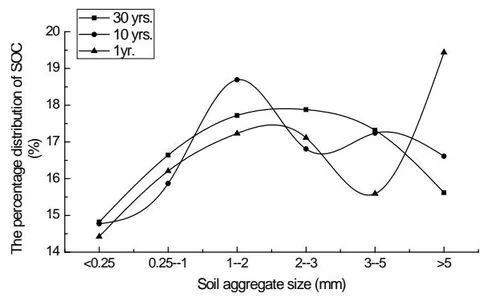
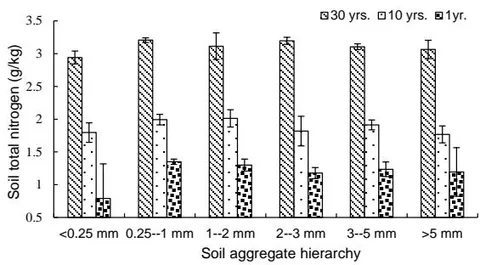
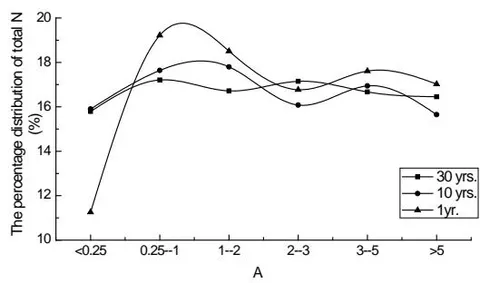
Fig. 2: Effect of restoration years on SOC and TN for different aggregate sizes
c) The distribution of soil microbial parameters at different aggregate sizes
i. Soil microbial biomass
The concentrations of , and at different grain sizes increases with length of grassland succession (Fig. 3 (a) and (e)). The situation with is different where it had the highest value in a 10 year natural grassland (Fig. 3 (c)).
Under a 30 year natural grassland, the percentage of (18.59) was greatest for a micro-aggregate size of <0.25 mm, as aggregate size increased, percentages dropped to a stable range between 15.68-16.56. At 10 years, a grain size of 1-2 mm showed the greatest percentage of (18.4), which was a rapid increase from <0.25. The percentage of for other particle sizes remained at a stable level between 16.72-17.61 (Fig 3 (b)). The curve of versus aggregate size for a recently abandoned grassland fluctuated greatly. There was a significant decrease in percentage of in 2-3 mm versus 1-2, 3-5 and >5 mm. In a 30-year natural grassland, the percentage of remained stable between 14.99 and 18.48 for the various aggregate sizes. As soil aggregate size increased, the distribution of in 1- and 10-year grassland showed a rising tendency and declining trend, respectively (Fig 3 (d)). The percentage of in different aggregate sizes for 10- and 30-year natural grassland remained stable. Whereas, for the highest percentage occurring in aggregate sizes of 2-3 mm, the 1-year curve showed a "normal distribution" which was significantly enhanced from 0.25-1 mm and rapidly declined at 2-3 mm (Fig 3 (f)).
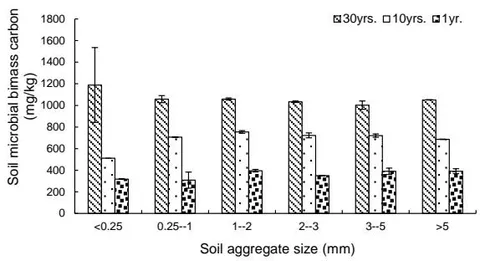
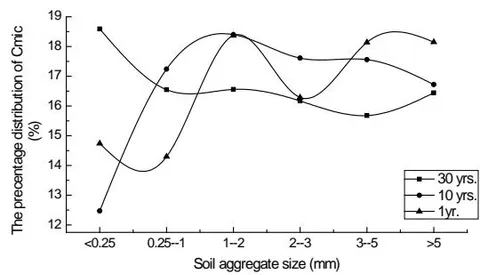
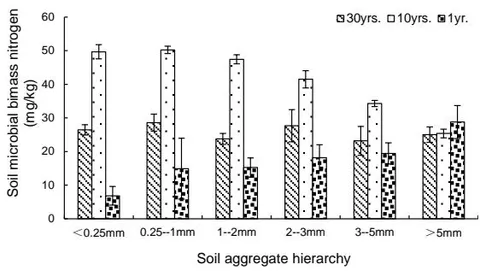
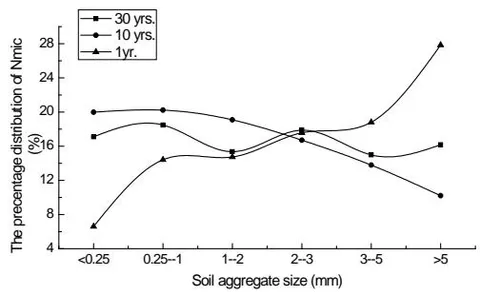
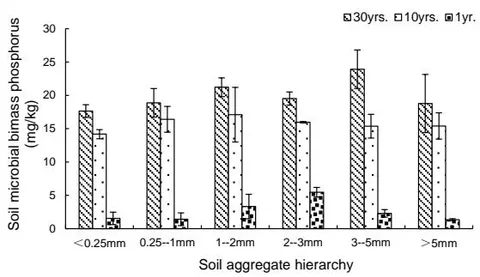
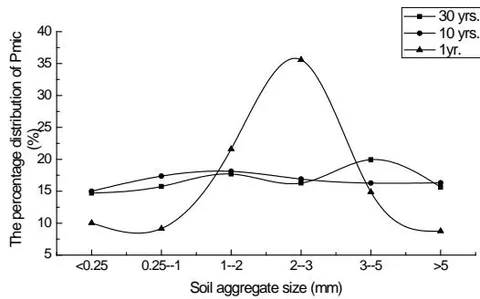
Fig. 3: Effect of restoration years on Cmic, Nmic and Pmic in different aggregate sizes
d) Soil microbial basal respiration and metabolic quotient
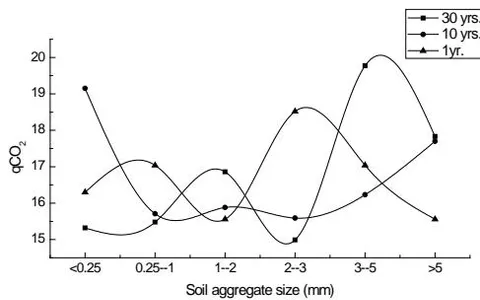
Soil microbial basal respiration (SBR) was enhanced as the successional years increased (Fig.4(a)). For a grassland abandoned for 1 year, the percentage of SBR in <0.25 and 0.25-1 mm was lower than in other aggregate sizes. SBR increased with aggregate size, the highest occurring between 3-5 mm. The curve of SBR for a 30-year natural grassland for different aggregate size classes fluctuated, it was the highest in 3-5 mm and lowest in 2-3 mm. However, the percentage at 10 years increased with soil aggregate size (Fig.4 (b)). Soil microbial metabolic quotient ( ) among the aggregate size classes had the opposite reaction as restoration years increased (Fig.4 (c)). In a grassland abandoned for 10 years, the percentage of , in aggregate size classes of 0.25-1, 1-2 and 2-3 mm, was lower than in the micro-aggregate (<0.25 mm) and macro-aggregate (3-5 mm and >5 mm) classes (Fig.4 (d)).
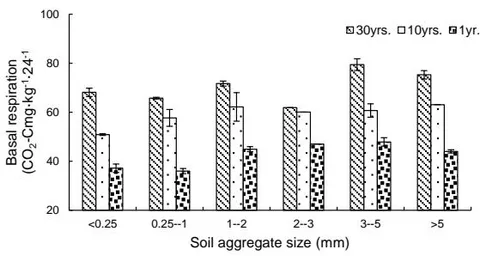
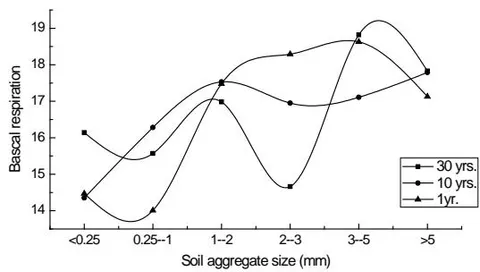
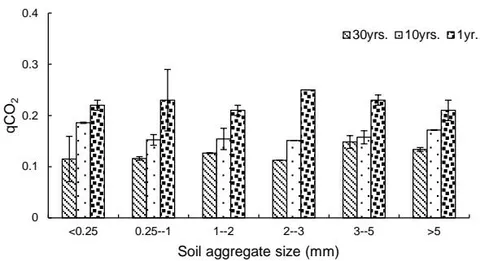
(b) The percent distribution of SBR in soil aggregate sizes (c) The distribution of qCO2 for different grassland restoration years;
(d) The percent distribution of qCO2 in soil aggregate sizes
Fig. 4: Effect of restoration years on SBR and qCO2 in different aggregate sizes e) The ratios of C/N, and Table 3: The ratios of C/N, and for different aggregate sizes
| Succesional years | Size classes (mm) | C/N | ||
| 30 | <0.25 | 8.42 | 67.38 | 44.92 |
| 0.25--1 | 8.67 | 56.05 | 37.03 | |
| 1--2 | 9.51 | 49.89 | 44.57 | |
| 2--3 | 9.35 | 52.98 | 37.37 | |
| 3--5 | 9.32 | 41.93 | 43.24 | |
| >5 | 8.52 | 56.01 | 42.02 | |
| Mean | 8.97 | 54.04 | 41.53 | |
| 10 | <0.25 | 8.95 | 36.09 | 10.30 |
| 0.25--1 | 8.67 | 43.11 | 14.08 | |
| 1--2 | 10.12 | 44.13 | 15.91 | |
| 2--3 | 10.08 | 45.25 | 17.41 | |
| 3--5 | 9.81 | 46.87 | 21.02 | |
| >5 | 10.23 | 44.53 | 27.04 | |
| Mean | 9.64 | 43.33 | 17.62 | |
| 1 | <0.25 | 10.40 | 206.01 | 46.49 |
| 0.25--1 | 6.85 | 218.87 | 20.67 | |
| 1--2 | 7.56 | 119.22 | 25.96 | |
| 2--3 | 8.29 | 64.21 | 19.32 | |
| 3--5 | 7.19 | 170.75 | 20.10 | |
| >5 | 9.28 | 290.95 | 13.58 | |
| Mean | 8.26 | 178.34 | 24.35 |
The ratios of C/N, and for the different aggregate sizes in the three successional periods were shown in Table 3. The greatest ratios of C/N, and were exhibited in the 10 year, 30 year and 1 year grasslands, respectively.
For the 10- and 30-year natural successional grasslands, the ratios of C/N in aggregate size of 1-2, 2-3 and 3-5 mm were higher than the others. The ratios of in grassland under succession for 30 years was greater in <0.25, 0.25-1 and >5 mm and were between 43.11-46.25 in grassland under succession for 10 years, expect <0.25 mm which had the lowest value. For a grassland under restoration for one year, the ratios show a V shaped distribution among the soil aggregate sizes, with the lowest ratio occurring in 2-3 mm. The ratio of in grassland that was in a natural state for 30 years was maintained at a stable level (37.03-42.02), but, at 10 years, the ratio increased as soil aggregate size increased. For a grassland and lowest for , the other ratios were abandoned for 1 year, the ratio was greatest for between 9.32 - 25.96.
f) The
| SOC | Total N | NO3-N | NH4-N | Ap-K | Ap-P | C/N | |
| 0.965** | 0.964** | 0.155 | -0.269 | 0.087 | 0.574* | 0.259 | |
| 0.268 | 0.206 | -0.704** | -0.106 | 0.046 | 0.035 | 0.312 | |
| 0.933** | 0.883** | -0.106 | -0.208 | 0.406 | 0.677** | 0.422 | |
| SBR | 0.910** | 0.882** | 0.046 | -0.098 | 0.207 | 0.672** | 0.326 |
| -0.932** | -0.906** | 0.035 | 0.395 | -0.267 | -0.473** | -0.463 |
Significant correlations were found between soil microbial properties and chemical characteristics. As Table 4 shows, a correlation exists among the soil microbial properties that were significantly correlated with SOC, TN and Ap-P. did not relate to SBR and , and only correlated with and were significantly correlated with SBR, and , (p<0.01). The ratio of was negatively correlated with (R=-0.638, p<0.01), (R=-507, p<0.05), (R=-0.833, p<0.01) and SBR (R=-0.727, p<0.01), and positively correlated with (R=0.635, p<0.01).
| SBR | |||||||
| 1 | |||||||
| 0.250 | 1 | ||||||
| 0.903** | 0.486** | 1 | |||||
| SBR | 0.917** | 0.305 | 0.933** | 1 | |||
| 0.954** | -0.414 | -0.901** | 0.841** | 1 | |||
| 0.593** | 0.548** | 0.369 | 0.472* | -0.463 | 1 | ||
| -0.638** | -0.507* | -0.833** | -0.727** | 0.635** | 0.142 | 1 |
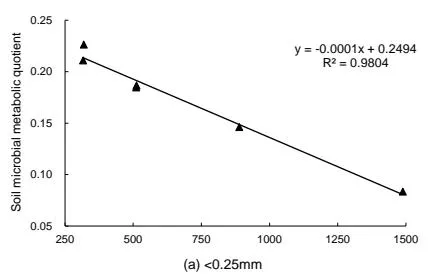
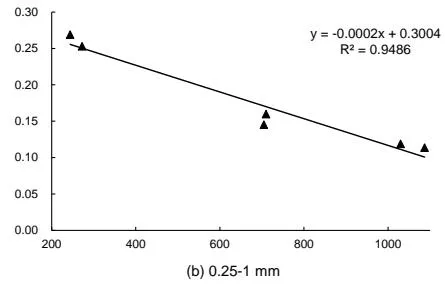
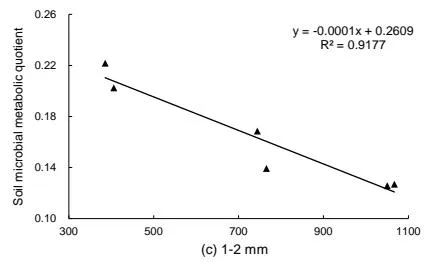
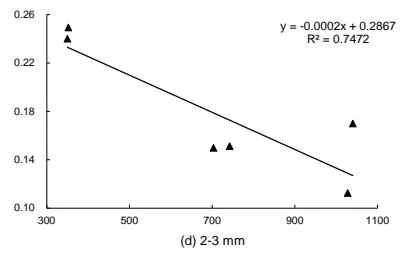
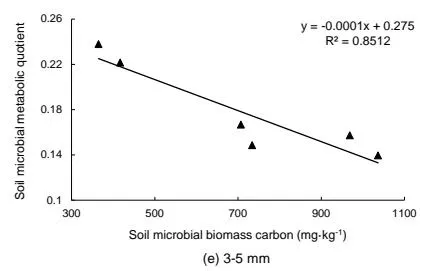
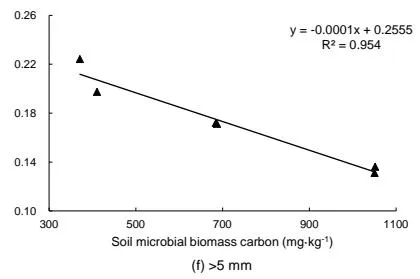
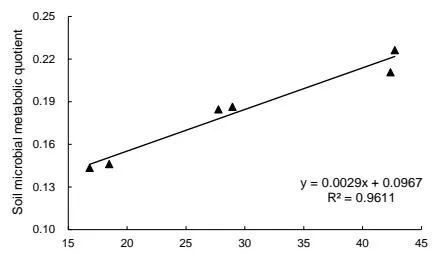
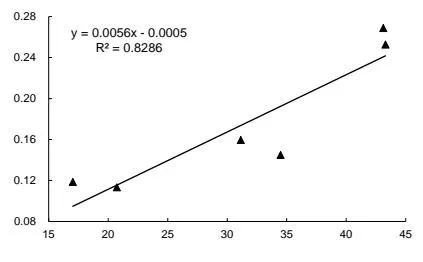
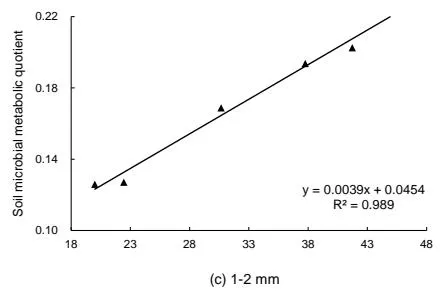
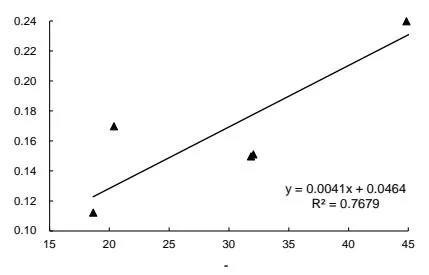
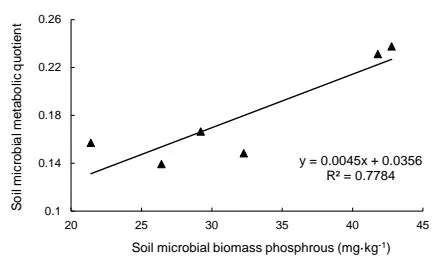
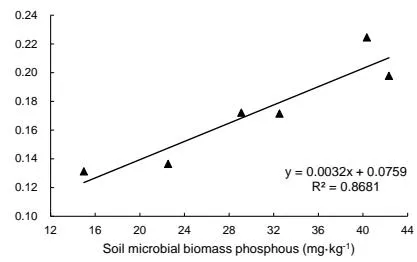
Table 5 shows that soil microbial metabolic quotient ( ) was positively related to (R=0.954) and negatively correlated to (R=-0.901), the correlation ratios were significant (p<0.01). The correlation between and , and in different aggregate sizes is shown in Figures 5 and 6. The correlation coefficients for and , and in <0.25, 0.25-1, 1-2 and >5 mm were higher (0.9177-0.9804, 0.8288-0.989) than in 2-3 (0.7427, 0.7679) and 3-5mm (Fig.5 (d) and (f)).
IV. DISCUSSION
Soil microbial parameters are indicators of soil quality and can be used to evaluate the success of revegetation in disturbed soil ecosystems (An, et al., 2009). Soil microbial biomass, basal respiration and metabolic quotient have been previously considered the most sensitive parameters for evaluating natural and degraded systems (Chen, et al., 2000; Dick et al., 1996; Bolinder et al., 1999; An et al., 2009). The microbial parameters measured in this study were measured at different aggregate sizes, and used to quantify soil quality differences under different successional stages or lengths of revegetation. In the present study, SOC, TN and Ap-P (chemical characteristics); Inv., Alk-P (soil enzyme activities); and (soil microbial biomass) increased with an increase in restoration years. Natural grassland flourished when grazing was prohibited. After the grassland was protected with fences, plant biomass and height increased, with a concommittal increase in soil organic matter.
The arrangement of the soil aggregates and their stability had a large influence on soil properties (Lynch and Bragg, 1985). The composition of the soil aggregates influenced the amount of soil organic matter, which in return affected the soil aggregate structure and stability by functioning as a bonding agent between mineral soil particles (Haynes and Beare, 1997; Chevallier, et al., 2004; Diaz, et al., 1994). Soil organic matter protects the soil surface against raindrop impact, improves water infiltration and impacts the hydrophobic characteristics that reduce wetting rates and slaking (Angers, et al., 1998). In 10- and 30-year natural grassland, the amount of was greatest in mm, then and lastly mm, respectively. In grassland that was abandoned for 1 year, the amount of was greatest in in 1-2, then 3-5 and, lastly >5 mm. Micro-aggregate size impacted accumulation, the effect of accumulation increased as the restoration years increased.
Soil microbial biomass contributed, with a significant portion in the active pools of SOC and TN. Soil microbial biomass C is one of the comprehensive indicators which reflect soil nutrient availability, biological activity and distribution of microorganism (An et al., 2009). It is the dynamic part of the soil carbon pool, which indicates the condition of soil organic matter accumulation (He, et al. 1997; Insam and Domsch, 1998). The soil microbial community influences soil mineralization and immobilization processes. The vegetative species and composition change as the vegetation restoration years increase, which impacts the soil microbial community in a direct way. An extensive root system provides the most improvement in soil structure by binding macro-aggregates to fine roots and VAM fungal hyphae and by binding micro-aggregates with adhesive bacterial metabolic products. (Lynch and Bragg, 1985; Carter, 1986; Perfect et al., 1990). Carbon input is the limiting factor in production of soil microbial biomass (Lynch and Panting, 1980; Insam & Haselwandter, 1989). The natural grassland with 30 years of restoration has a species-rich plant community that protects soil from physical disturbance (Pérès, et al., 2013), and higher soil organic matter supports an abundant carbon source for the growth of microorganisms and metabolism (Six, et al., 1999 and 2000a; Anderson and Gray, 1990), which results in the highest amounts of and . The percentage of at different aggregate sizes was stable (Six, et al., 2000b).
Anderson and Domsch (1985) proposed that the ratio of soil basal respiration to microbial biomass (soil microbial metabolic quotient or ), was the most sensitive indicator of quantitative and qualitative changes in microbial communities caused by various management systems (Insam et al., 1989). It was identified as the most important parameter in analyzing vegetation and soil microbial characteristics (Bastida et al., 2008; An et al., 2009). Soil respiration relies on a suite of complex processes contributing to efflux from soil surface, mainly from plant roots and micro-organisms (Jia, et al., 2006; An et al., 2009). Many studies showed the changes in soil respiration and soil microbiological properties with succession (Schafer, et al., 1979; Mathes and Schriefer, 1985; Stroo and Jencks, 1982; Insam & Hasel wandter, 1989). In this study, soil basal respiration was enhanced as natural restoration years increased with the highest concentrations found at the macro-aggregate level. The findings of Insam and Haselwandtere (1989) on two 50-year-old soil chronosequences on reclamation sites are similar. However, soil microbial metabolic quotient ( ) declined as vegetation restoration years increased. The percentage of in micro-aggregate sizes was lower than in macro-aggregate sizes, the distributions of SOC and TN in different aggregate sizes was similar. Because was negatively correlated with SOC and total N, the decrease in with time for the vegetated areas at different aggregate sizes resulted in competition for the available carbon source, which seemed to favor aggregate classes that needed the least amount of energy for maintenance and growth (Insam and Haselwandter, 1989). In the current study, relationships existed between and SOC, TN, Ap-P, , and SBR. Especially for and , the ratios in 2-3 mm were lowest (0.7472 and 0.7679, respectively). Wardle (1992) indicated that a lower microbial biomass concentration can be characteristic of disturbance, and it is an obvious factor that induces a rise in . A higher and a lower microbial biomass may both occur late in ecosystem succession, and the relationship between the two reflects their dual response to underlying stress (Wardle & Ghani, 1995). The result demonstrates that 2-3 mm is the relative stable aggregate size class in ecosystem succession.
V. CONCLUSION
Loess plateau ecosystems are suffering serious environmental problems including natural grassland degradation due to soil and water erosion. This study shows that grassland has a positive effect on soil status as indicated by an increase in the concentration of soil nutrients and microbial biomass. As grassland restoration years increased, soil microbial biomass carbon, phosphorus and basal respiration increased. Soil microbial metabolic quotient ( ) an alternative measure that changes when microbial biomass responses to disturbances, is significantly correlated to and , the lowest ratios illustrated that 2-3 mm was the stablest aggregate size in the process of ecological restoration.
ACKNOWLEDGEMENTS
This study was supported by Key Laboratory Open Project Fund (A314021402-1707), the National Natural Sciences Foundation of China (41571260, 41807060), and National Special Research and Development Project during the Thirty Five-year Plan Period (2017YFC0504702).